BPC-157
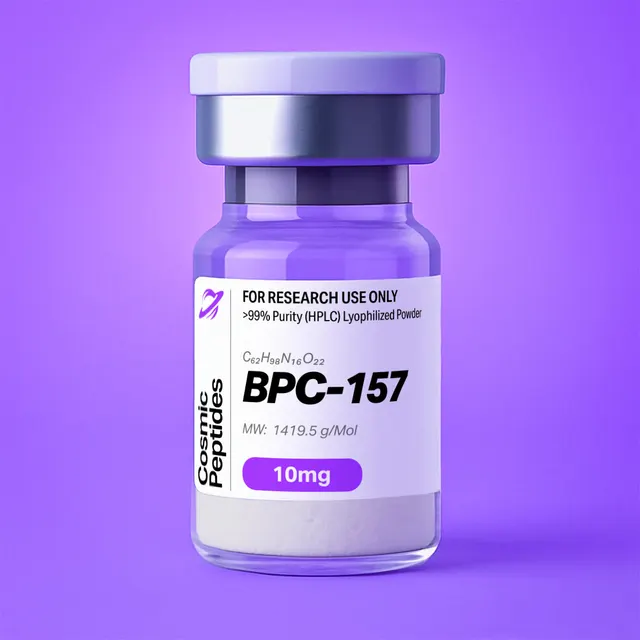
BPC-157
Commonly researched with these items
Patent-pending lot tracking: Complete transparency from production to vial.
| CAS Number | 137525-51-0 |
|---|---|
| Molecular Formula | C62H98N16O22 |
| Molecular Weight | 1419.54 g/Mol |
| Purity | 99.7% |
| Lot Number | 26107 |
| Quantity | 10.61mg |
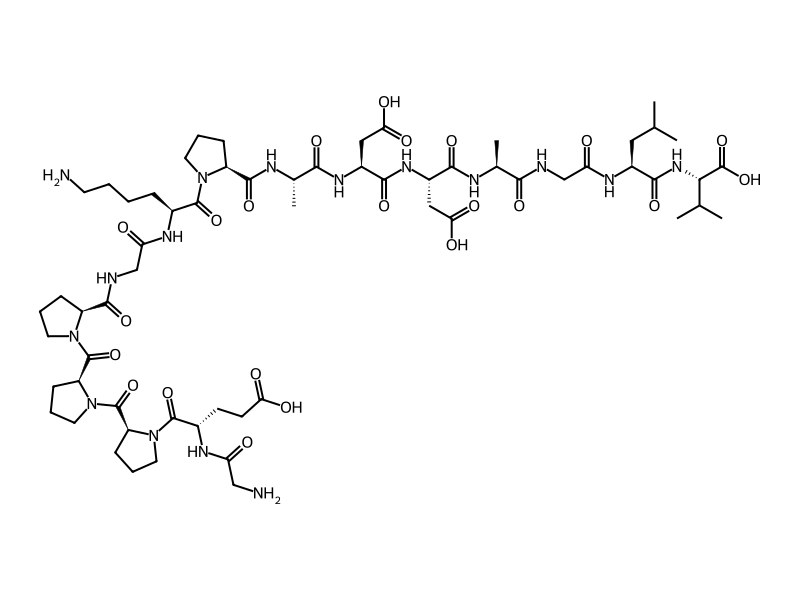
| Sequence | Gly-Glu-Pro-Pro-Pro-Gly-Lys-Pro-Ala-Asp-Asp-Ala-Gly-Leu-Val |
BPC-157: The Proline-Rich Gastric Pentadecapeptide GEPPPGKPADDAGLV
Disclaimer
Products described here are supplied for research use only and are not intended for diagnostic, therapeutic, or clinical application. All statements regarding biological activity reflect preclinical and in vitro findings exclusively and have not been evaluated by the U.S. Food and Drug Administration. These materials and related content are provided for educational and investigational purposes only and are intended solely for qualified researchers in laboratory and academic settings.
Key Facts
- Compound class
- Linear, unmodified pentadecapeptide; a synthetic partial sequence of the gastric-juice protein body protection compound (BPC)
- Sequence / structure
H-Gly-Glu-Pro-Pro-Pro-Gly-Lys-Pro-Ala-Asp-Asp-Ala-Gly-Leu-Val-OH(one-letter code:GEPPPGKPADDAGLV), all chiral residues in the L-configuration, free N-terminal amine and free C-terminal acid- Molecular formula
- C62H98N16O22
- Molecular weight
- 1419.54 g/mol (average, free peptide); monoisotopic mass 1418.7042 Da
- CAS number
- 137525-51-0
- PubChem CID
- 9941957
- Other designations
- BPC 157, Bepecin, PL 14736, PL-10, PLD-116 (synonyms listed in PubChem)
- Physical form as supplied
- Lyophilized powder
- Lot traceability
- Every unit is tied to a tracked lot; the lot number, recorded purity and verified quantity of the lot on sale are shown live on this page, with its certificate of analysis.
Molecular Identity and Classification
BPC-157 is the pentadecapeptide glycyl-glutamyl-prolyl-prolyl-prolyl-glycyl-lysyl-prolyl-alanyl-aspartyl-aspartyl-alanyl-glycyl-leucyl-valine, written H-GEPPPGKPADDAGLV-OH. It is linear, with no disulfide bonds, terminal capping groups, non-proteinogenic residues or post-translational modifications: every one of its fifteen residues is a standard L-amino acid (or the achiral glycine), joined by ordinary amide bonds from a free N-terminal glycine amine to a free C-terminal valine carboxylic acid.
The molecular formula is C62H98N16O22. Its average molecular weight is 1419.54 g/mol when calculated with conventional atomic weights (PubChem rounds it to 1419.5 g/mol). The monoisotopic mass, the value that matters for high-resolution mass spectrometry, is 1418.7042 Da. The compound is registered under CAS number 137525-51-0 and appears in PubChem as compound 9941957, where the depositor synonyms include BPC 157, Bepecin, PL 14736, PL-10 and PLD-116.
The name "BPC" stands for body protection compound, the term Sikirić and colleagues at the University of Zagreb used in 1993 for a gastric-juice protein fraction of apparent mass Mr 40,000 (about 40 kDa). The fifteen-residue sequence was described as a partial sequence of that protein, and 157 belongs to the laboratory designation of the synthetic fragment. Early papers group the synthetic fragments as "PL-10" substances; work from the 2000s uses the designation PL 14736 for exactly this sequence; and a 2025 literature and patent review by Józwiak and colleagues surveys the patent filings covering it. Because the PL-10 series contained more than one peptide, the sequence printed in each paper should be checked.
At fifteen residues it is too short to fold into a stable tertiary structure, yet long enough to carry distinct structural regions: an N-terminal triproline segment, a central Lys-Pro motif, an acidic Asp-Asp pair and a short hydrophobic C-terminus. Four acidic groups (Glu2, Asp10, Asp11 and the C-terminal carboxylate) outnumber the two basic groups (the N-terminal amine and Lys7), making it an unusually acidic research peptide and shaping its solubility, chromatography and ionization.
Structure and Chemical Features
| Residues | Segment | Chemical character | Analytical consequence |
|---|---|---|---|
| 1–2 | Gly-Glu | Free α-amine (pKa about 8–9.6) and the first acidic side chain | N-terminal amine is the main site for amine-reactive labelling reagents |
| 3–6 | Pro-Pro-Pro-Gly | Triproline run with high polyproline II (PPII) propensity; three tertiary amide bonds | Multiple cis/trans prolyl isomers; doubled or broadened NMR signals |
| 7–8 | Lys-Pro | The only basic side chain, followed by a fourth proline | Preferred proton site in ESI; favoured cleavage N-terminal to Pro8 in MS/MS |
| 9–12 | Ala-Asp-Asp-Ala | Acidic pair with two β-carboxylates | Dominates net negative charge; aspartimide-prone during Fmoc synthesis |
| 13–15 | Gly-Leu-Val | Hydrophobic C-terminal tail ending in a free carboxylic acid | Main hydrophobic contact for reversed-phase retention |
The proline content. Four of the fifteen residues (27%) are proline, at positions 3, 4, 5 and 8. Proline is the only proteinogenic amino acid whose side chain is bonded back to its own backbone nitrogen, forming a pyrrolidine ring that fixes the backbone dihedral angle φ near −65°. Each of the four X–Pro bonds is a tertiary amide with no N–H, so it cannot donate a hydrogen bond, and the energetic preference for the trans over the cis isomer is small enough that several percent to tens of percent of each bond can populate the cis form in water. With four such bonds the peptide can in principle exist as up to 24 = 16 prolyl isomers that interconvert on a timescale of seconds to minutes at room temperature, as reviewed by Wedemeyer, Welker and Scheraga. This is the single most important structural fact for interpreting BPC-157 spectra: minor sets of resonances in 1H or 13C NMR, and occasionally peak broadening at low column temperature in HPLC, are expected properties of the pure compound and not, by themselves, evidence of impurity.
Polyproline II character. Proline-rich stretches in short peptides tend to adopt the left-handed, extended polyproline II helix, with about three residues per turn and a rise of roughly 3.1 Å per residue. Adzhubei, Sternberg and Makarov's review notes that unfolded peptides are rich in PPII and that proline-rich recognition sites tend to adopt it. For BPC-157 that implies a locally rigid, extended Pro3-Pro4-Pro5 rod with Gly6 and Gly13 as flexible hinges. In circular dichroism, PPII shows a strong negative band near 205 nm and a weak positive band near 228 nm.
Charge and ionizable groups. The peptide carries six ionizable groups: the N-terminal α-amine, the Lys7 ε-amine (pKa about 10.5), the Glu2 γ-carboxylate (about 4.2), the Asp10 and Asp11 β-carboxylates (about 3.9 each) and the C-terminal carboxylate (about 2.3 to 3.5). At pH 7 the two amines are protonated and all four carboxylic acids deprotonated, giving a net charge of approximately −2. The calculated isoelectric point falls between about 3.7 and 4.2 depending on the pKa set used, so the peptide is least soluble, and most prone to adsorb or aggregate, near pH 4. PubChem's computed descriptors (XLogP3 −9, polar surface area 573 Å2) describe an extremely polar molecule.
What the sequence lacks. BPC-157 contains no cysteine, methionine, tryptophan, tyrosine, phenylalanine, histidine, asparagine, glutamine, serine or threonine. There is therefore no thiol or thioether to oxidize, no aromatic chromophore, no metal-binding imidazole and no deamidation site. The principal chemical liabilities are confined to the Asp-Asp pair (isomerization through a succinimide intermediate) and to slow hydrolysis of peptide bonds at pH extremes.
Synthesis and Manufacturing Chemistry
BPC-157 is made by solid-phase peptide synthesis (SPPS), introduced by Merrifield in 1963, using the base-labile 9-fluorenylmethoxycarbonyl (Fmoc) α-amine protecting group of Carpino and Han (1972). For a C-terminal free acid the chain is started on an acid-labile resin such as 2-chlorotrityl chloride or Wang resin preloaded with Fmoc-Val, and fourteen cycles of Fmoc removal (typically 20% piperidine in dimethylformamide) and coupling (DIC/Oxyma, HBTU or HATU) build the chain towards the N-terminus.
Four side chains need protection: Glu2 and the two aspartates as tert-butyl esters (Fmoc-Glu(OtBu)-OH, Fmoc-Asp(OtBu)-OH) and Lys7 as the Boc carbamate (Fmoc-Lys(Boc)-OH). Final cleavage in trifluoroacetic acid (TFA) with water and triisopropylsilane as scavengers releases the peptide and removes all protecting groups in one step; the crude product is precipitated in cold ether, purified by preparative reversed-phase HPLC and lyophilized.
Four challenges are specific to this sequence:
- Couplings onto proline. Pro3, Pro4, Pro5 and Pro8 present secondary amines, less nucleophilic and more hindered than primary amines, so the Glu-onto-Pro, Pro-onto-Pro and Lys-onto-Pro steps are often double-coupled or run with a stronger activator. Because the Kaiser (ninhydrin) test does not give its usual blue colour with a secondary amine, completeness is checked with the chloranil or isatin test instead.
- Aspartimide formation. Repeated exposure to piperidine can drive the backbone nitrogen of the residue following an aspartate to attack the Asp side-chain ester, forming a five-membered succinimide (aspartimide). Ring opening then gives a mixture of α- and β-aspartyl peptides and their D-epimers, all with the same mass as the target. Mergler and colleagues showed that the extent depends strongly on the residue after Asp and on the side-chain ester. In BPC-157 the Asp10-Asp11 and Asp11-Ala12 junctions are less prone than the notorious Asp-Gly motif, but remain the most likely origin of isobaric impurities; bulkier esters, additives such as Oxyma in the deprotection solution, or shorter piperidine exposure suppress them.
- Diketopiperazine at the dipeptide stage. After Fmoc removal from resin-bound Leu-Val, the free amine can cyclize onto the ester linkage and release cyclo(Leu-Val), truncating the chain. The hindered 2-chlorotrityl linker and prompt coupling of Gly13 keep this low.
- Deletion sequences. Incomplete coupling in the Pro-Pro-Pro region yields des-Pro peptides that differ from the target by exactly 97.0528 Da (one proline residue). They co-elute closely with the main peak and are best detected by mass.
Counterions. Because TFA is used in cleavage and in preparative HPLC, synthetic BPC-157 is commonly obtained as a trifluoroacetate salt, and PubChem lists "BPC 157 trifluoroacetate" among its synonyms; the two basic sites can each carry one trifluoroacetate. Material can be exchanged into acetate or chloride by ion exchange or repeated lyophilization from dilute acid. The counterion changes the mass of peptide per milligram of powder, as the calculation below shows.
Analytical Characterization
Reversed-phase HPLC. Purity is measured by reversed-phase HPLC on C18 columns with water/acetonitrile gradients containing 0.1% TFA or formic acid, following the principles summarized by Mant and colleagues. Having no aromatic residue, BPC-157 has essentially no absorbance at 280 nm; detection relies on the amide bonds at 210–220 nm (most often 214 nm). Aromatic impurities such as Fmoc-derived material absorb disproportionately at 214 nm and can make a chromatogram look worse than the mass balance suggests. Retention increases markedly at low pH, where the four carboxylic acids are protonated, and column temperatures of 40–60 °C sharpen peaks by accelerating prolyl cis/trans interconversion.
Mass spectrometry. Electrospray ionization confirms identity. The expected ions, calculated from the monoisotopic mass of 1418.7042 Da, are listed below. In positive mode the doubly protonated ion is usually the base peak, with protons on the N-terminal amine and Lys7; the triply charged ion is weak because a third proton has no strongly basic site. Being acidic, the molecule also ionizes well in negative mode, giving a strong [M−2H]2− ion. With 62 carbon atoms the first 13C isotope peak (M+1) is about 75% as intense as the monoisotopic peak, so in the [M+2H]2+ envelope the peaks at m/z 710.36 and 710.86 are nearly equal in height: the M+1 peak must not be mistaken for the monoisotopic ion when mass error is calculated.
| Ion | m/z (monoisotopic) | Notes |
|---|---|---|
| [M+H]+ | 1419.7114 | Prominent in MALDI; weaker in ESI |
| [M+2H]2+ | 710.3594 | Usually the base peak in positive ESI |
| [M+3H]3+ | 473.9087 | Weak; only two strongly basic sites |
| [M+Na]+ | 1441.6934 | Common adduct from glass or buffer sodium |
| [M−H]− | 1417.6969 | Negative-mode ESI |
| [M−2H]2− | 708.3448 | Strong in negative mode, owing to four carboxylates |
Tandem MS fragmentation. Collision-induced dissociation of [M+2H]2+ follows the "proline effect": cleavage of the amide bond on the N-terminal side of a proline is strongly favoured. Breci and colleagues' analysis of a large database of peptide spectra found that this enhancement is greatest when the residue before proline is Val, His, Asp, Ile or Leu, and weakest when it is Gly or Pro. In BPC-157 the bond N-terminal to Pro8 (Lys-Pro) is therefore expected to be the most productive cleavage site, giving the complementary pair b7 (GEPPPGK, m/z 663.346) and y8 (PADDAGLV, m/z 757.373), while cleavages inside the Pro-Pro-Pro run should be weaker. Other diagnostic singly charged fragments are b2 (GE, 187.071), y2 (LV, 231.170), y3 (GLV, 288.192), y4 (AGLV, 359.229), y6 (DDAGLV, 589.283) and y12 (PPGKPADDAGLV, 1136.595). Aspartate also favours cleavage C-terminal to itself (the "aspartic acid effect"), so b10 (946.463) and b11 (1061.490) are worth adding to a targeted method.
Distinguishing isobaric impurities. Aspartimide-derived β-aspartyl and D-aspartyl isomers have the same mass as BPC-157, so MS alone cannot exclude them; they are resolved chromatographically and identified against prepared reference isomers or by chiral amino-acid analysis. The succinimide intermediate itself appears at −18.0106 Da (loss of water) from the parent.
Amino-acid analysis. After 6 M HCl hydrolysis the expected composition is Gly 3, Pro 4, Ala 2, Asx 2, Glx 1, Lys 1, Leu 1 and Val 1. Proline is a secondary amine and does not react with o-phthalaldehyde, so OPA methods need a second reagent such as FMOC-Cl, or ninhydrin detection at 440 nm, to quantify it. Pro-Pro bonds hydrolyse slowly, so a short hydrolysis lowers the apparent proline count.
Purity versus peptide content, with a worked calculation. HPLC purity reports what fraction of the UV-absorbing material is BPC-157. Peptide content reports what fraction of the weighed powder is peptide rather than counterions, water and salts. With two basic sites, the counterion correction is easy to estimate:
| Form | Formula weight | Peptide fraction by mass |
|---|---|---|
| Free peptide (zwitterion) | 1419.54 g/mol | 100% |
| Monoacetate (+1 CH3COOH, 60.05) | 1479.6 g/mol | 95.9% |
| Diacetate (+2 × 60.05) | 1539.6 g/mol | 92.2% |
| Mono-trifluoroacetate (+1 CF3COOH, 114.02) | 1533.6 g/mol | 92.6% |
| Bis-trifluoroacetate (+2 × 114.02) | 1647.6 g/mol | 86.2% |
A bis-trifluoroacetate powder with 5% bound water would therefore contain only about 82% peptide by weight even at 99% HPLC purity, so a nominally 1.0 mM solution made by weight alone would be nearly 20% low. Where exact concentrations are required, peptide content should be determined by amino-acid analysis, quantitative NMR or nitrogen analysis, and counterion content by ion chromatography or 19F NMR for trifluoroacetate.
Physicochemical Properties
| Property | Value | Notes |
|---|---|---|
| Molecular formula | C62H98N16O22 | Without counterions or water |
| Average molecular weight | 1419.54 g/mol | PubChem CID 9941957 lists 1419.5 |
| Monoisotopic mass | 1418.7042 Da | PubChem exact mass 1418.70415882 |
| Residues | 15 | Gly 3, Pro 4, Ala 2, Asp 2, Glu 1, Lys 1, Leu 1, Val 1 |
| Net charge at pH 7 | approximately −2 | Four carboxylates, two ammonium groups |
| Isoelectric point | about 3.7–4.2 (calculated) | Acidic; minimum solubility near pH 4 |
| XLogP3 | −9 | Computed (PubChem); extremely hydrophilic |
| Topological polar surface area | 573 Å2 | Computed (PubChem) |
| Hydrogen-bond donors / acceptors | 16 / 24 | Computed (PubChem) |
| Rotatable bonds | 39 | Computed (PubChem) |
| GRAVY (Kyte–Doolittle) | −0.69 | Calculated from sequence; net hydrophilic |
| Prolyl bonds | 4 (Glu–Pro, Pro–Pro, Pro–Pro, Lys–Pro) | Up to 16 cis/trans isomers in solution |
| UV absorbance | Peptide bond only (about 214 nm) | No Trp, Tyr or Phe; no 280 nm signal |
| Oxidation-sensitive residues | None | No Cys, Met or Trp |
| Solubility | Readily soluble in water and neutral aqueous buffers | Typical for a charged, hydrophilic 15-mer |
A polar surface area above 500 Å2 and 16 hydrogen-bond donors place the peptide far outside the range for passive diffusion across lipid bilayers, so cell-based results have to be interpreted in terms of cell-surface interactions, carrier-mediated uptake or endocytosis.
Stability in buffer does not carry over to biological matrices: Cox, Miller and Eichner (2017) found in their in vitro plasma incubations that BPC-157 is converted to a stable metabolite, and Tian and colleagues (2023) identified nine metabolites from two in vitro incubation models, eight of them formed by amide-bond cleavage. Serum-containing culture medium should therefore be assumed to degrade the peptide.
Research Context
The in vitro literature asks a tractable question: which signalling pathways change when cultured cells are exposed to the peptide, and how do those changes track migration, spreading and tube formation? No specific receptor for BPC-157 has been identified, which is why many studies measure several pathways in parallel.
Fibroblast Migration and the FAK–Paxillin Axis
Chang and colleagues (2011) worked with cultured tendon fibroblasts. In the cell-culture part of that report, exposure to BPC-157 left proliferation unchanged in an MTT assay, raised the fraction of cells still viable after a hydrogen peroxide challenge, and increased migration in transwell filter assays and spreading on culture dishes in a concentration-dependent manner. Phalloidin staining showed increased F-actin formation, and immunoblotting showed concentration-dependent increases in the phosphorylation of focal adhesion kinase (FAK) and paxillin without a change in total protein. FAK and paxillin are core components of focal adhesions, the structures that couple integrins to the actin cytoskeleton, and their phosphorylation is a standard read-out of adhesion-complex turnover. The split between unchanged proliferation and increased motility is what makes this a cytoskeletal rather than a mitogenic observation.
A follow-up by the same group (Chang et al., 2014) screened exposed tendon fibroblasts by cDNA microarray and found the growth hormone receptor among the most strongly up-regulated transcripts, concentration- and time-dependently at both mRNA (RT-qPCR) and protein (Western blot) levels. Adding growth hormone to BPC-157-exposed cells increased proliferation (MTT, PCNA) and time-dependently activated Janus kinase 2 (JAK2), the kinase that couples the growth hormone receptor to STAT signalling. BPC-157 itself was not mitogenic here; it changed the cells' responsiveness to a second ligand.
Endothelial Cell Signalling
In the cultured-cell experiments of Huang and colleagues (2015), BPC-157 increased proliferation of human umbilical vein endothelial cells (HUVECs) (MTT, cell-cycle analysis), migration (transwell and scratch assays) and tube formation on basement-membrane matrix, raised VEGF-A expression, and changed the phosphorylation of ERK1/2 and the expression of their immediate-early targets c-Fos, c-Jun and Egr-1. Hsieh and colleagues (2017), by contrast, found that BPC-157 increased the mRNA and protein expression of vascular endothelial growth factor receptor 2 (VEGFR2) in endothelial cells without increasing VEGF-A, increased the rate of VEGFR2 internalization, and time-dependently activated the VEGFR2–Akt–eNOS pathway. Dynasore, an inhibitor of dynamin-dependent endocytosis, blocked the internalization, the pathway activation and the increase in tube formation, implicating receptor trafficking in the response. The discrepancy on VEGF-A shows why cell source, serum conditions and peptide salt form should be reported in full.
Hsieh and colleagues (2020) extended this to nitric oxide signalling: in endothelial cells BPC-157 raised intracellular nitric oxide (DAF-FM diacetate probe) and the phosphorylation of Src, caveolin-1 (Cav-1) and endothelial nitric oxide synthase (eNOS), and a Src inhibitor abolished these effects, placing Src upstream. Co-immunoprecipitation showed reduced Cav-1–eNOS binding, consistent with the mechanism by which caveolin-1 holds eNOS inactive until released.
Epithelial Cells and Immediate-Early Genes
Tkalčević and colleagues (2007), working with the same sequence under the designation PL 14736, studied the immediate-early gene egr-1 in undifferentiated Caco-2 colorectal epithelial cells. PL 14736 induced egr-1 and its co-repressor nab2 (NGFI-A binding protein 2) more rapidly than the reference growth factor PDGF-BB. EGR-1, a zinc-finger transcription factor induced within minutes of many stimuli, is a convenient early-response marker. Earlier, Bódis and colleagues (1997) compared four synthesized PL-10 peptides in two isolated cell preparations: two of the four lowered the loss of viability in isolated gastric mucosal cells exposed to ethanol, while the same two had no measurable effect in a myeloma cell line (Sp2/0-Ag14). Such a split between two cell types in one assay format is an early in vitro argument against a general physicochemical effect on membranes.
Designing In Vitro Experiments
Common read-outs are kinase phosphorylation by immunoblot, transcripts by RT-qPCR, migration by transwell or gap-closure assays, F-actin by phalloidin, tube formation, nitric oxide by DAF-FM fluorescence and viability by MTT. For a peptide with no defined receptor, good practice includes full concentration–response series (commonly spanning nanomolar to low micromolar), time courses that separate minute-scale phosphorylation from hour-scale transcription, a scrambled-sequence peptide of identical composition as a specificity control, a vehicle matched for counterion (trifluoroacetate alone can alter cell proliferation, as Cornish and colleagues showed), and LC-MS confirmation that the intact peptide is still present in the medium at the end of the experiment, given the protease susceptibility seen in biological matrices.
Related Research Peptides Compared
BPC-157 is often studied alongside other short peptides with very different chemistry (free-peptide values).
| Property | BPC-157 | TB-500 | KPV |
|---|---|---|---|
| Sequence | GEPPPGKPADDAGLV | Ac-LKKTETQ-OH | KPV |
| Length | 15 residues | 7 residues | 3 residues |
| Molecular formula | C62H98N16O22 | C38H68N10O14 | C16H30N4O4 |
| Average molecular weight | 1419.54 g/mol | about 889 g/mol | 342.43 g/mol |
| Termini | Free amine, free acid | N-acetylated, free acid | Free amine, free acid |
| Net charge at pH 7 | about −2 | about 0 | about +1 |
| Proline residues | 4 | 0 | 1 |
| Aromatic residues | None | None | None |
TB-500 is an acetylated heptapeptide corresponding to the actin-binding region of thymosin β4, and BPC-157/TB-500 supplies both peptides together. Their monoisotopic masses differ by about 530 Da, so each component of a combined material is identified unambiguously by mass, and TB-500 is near-neutral at pH 7 where BPC-157 is doubly anionic, which is what separates them on a C18 gradient. KPV is a basic tripeptide, the C-terminal fragment of α-melanocyte-stimulating hormone; with only three residues, a free basic amine and two small hydrophobic side chains it presents far less hydrophobic surface than BPC-157 and is expected to elute much earlier on a reversed-phase column.
Laboratory Handling and Storage
Storage of the solid. Lyophilized BPC-157 is best stored tightly closed at −20 °C, protected from light and moisture, or at −80 °C for long-term reference material. Lyophilized peptide salts are hygroscopic: let a container taken from the freezer reach room temperature in a desiccator before opening, so atmospheric moisture does not condense on the cold powder and add to the weighed mass.
Preparing solutions. BPC-157 dissolves readily in high-purity water and in neutral buffers such as phosphate-buffered saline. If a powder dissolves slowly, a little dilute ammonium bicarbonate or ammonium hydroxide raises the pH away from the isoelectric region; unbuffered dilute acid near pH 4 is the worst choice, because there the net charge approaches zero and solubility is at a minimum. Stock solutions of 1–10 mM are typical; for cell work, filter through a 0.22 µm low-binding membrane, divide into single-use aliquots and freeze at −20 °C or −80 °C, avoiding repeated freeze–thaw cycles.
Solution stability. In solution the main chemical risks are Asp10/Asp11 isomerization through a succinimide intermediate, accelerated by elevated temperature and mildly basic pH, and slow amide hydrolysis at pH extremes. Without Cys, Met or Trp, oxidation is not a concern. In biological matrices proteolysis dominates, so time points should be planned around it.
Adsorption. At nanomolar to low micromolar concentrations peptides adsorb to plastic and glass; low-binding polypropylene ware and, where the design allows, a carrier protein in the assay buffer reduce the losses.
Verification. A quick LC-MS run of a stock solution, looking for [M+2H]2+ at m/z 710.36 (or [M−2H]2− at 708.34 in negative mode), confirms identity and integrity after storage. A new peak at −18 Da from the parent mass points to succinimide formation, and smaller fragments matching b- or y-ions point to hydrolysis.
Frequently Asked Research Questions
- What is BPC-157?
- BPC-157 is a synthetic linear pentadecapeptide with the sequence Gly-Glu-Pro-Pro-Pro-Gly-Lys-Pro-Ala-Asp-Asp-Ala-Gly-Leu-Val (GEPPPGKPADDAGLV), described as a partial sequence of body protection compound (BPC), a protein fraction isolated from gastric juice. Its molecular formula is C62H98N16O22 and its average molecular weight 1419.54 g/mol.
- What is the CAS number of BPC-157?
- BPC-157 is registered under CAS number 137525-51-0 and appears in PubChem as compound 9941957.
- What ions should I see for BPC-157 by mass spectrometry?
- In positive ESI the base peak is usually [M+2H]2+ at m/z 710.359, with [M+H]+ at 1419.711 and a weak [M+3H]3+ at 473.909. In negative ESI, [M−2H]2− appears at 708.345. The monoisotopic mass of the neutral peptide is 1418.7042 Da.
- Which MS/MS fragments identify BPC-157?
- Cleavage N-terminal to Pro8 is favoured by the proline effect, giving b7 at m/z 663.346 and y8 at 757.373. Useful additional ions include y2 (231.170), y3 (288.192), y4 (359.229) and y6 (589.283).
- Why does BPC-157 show no absorbance at 280 nm?
- The sequence contains no tryptophan, tyrosine or phenylalanine, the residues responsible for absorbance near 280 nm. HPLC detection relies on the peptide bonds at 210–220 nm, and concentrations cannot be determined from A280.
- Why does a pure BPC-157 sample give extra NMR signals?
- The peptide has four X–Pro bonds, each of which exists as slowly interconverting cis and trans isomers. Up to sixteen prolyl isomers can coexist in solution, producing minor resonance sets that are a property of the pure compound rather than an impurity.
- What is the difference between HPLC purity and peptide content?
- HPLC purity is the fraction of UV-absorbing material that is BPC-157. Peptide content is the fraction of the powder's mass that is peptide rather than counterions, water and salts. A bis-trifluoroacetate salt is only 86.2% peptide by mass before any water is counted, so molar work requires a peptide-content correction.
- Which impurities are typical of synthetic BPC-157?
- The most characteristic are des-Pro deletion peptides (−97.05 Da) from incomplete coupling in the Pro-Pro-Pro region, and isobaric β-aspartyl or D-aspartyl isomers from aspartimide formation at the Asp-Asp pair, which must be resolved chromatographically because they have the same mass.
- Which signalling pathways have been studied with BPC-157 in cultured cells?
- In vitro studies have measured FAK–paxillin and growth hormone receptor–JAK2 signalling in tendon fibroblasts; VEGFR2–Akt–eNOS, Src–caveolin-1–eNOS and ERK1/2 signalling in endothelial cells; and egr-1 induction in Caco-2 cells.
- How do I prepare a 1 mM stock of BPC-157?
- The free peptide has a molar mass of 1419.54 g/mol, so 1 mM is 1.42 mg of peptide per mL. Divide that figure by the peptide content of the powder: at 85% peptide content, 1.42 / 0.85 = 1.67 mg of powder per mL. Weighing 10.0 mg of free peptide corresponds to 7.04 µmol, which makes 7.04 mL of a 1 mM solution.
- Does BPC-157 survive in serum-containing culture medium?
- It should not be assumed to. In vitro metabolism studies report conversion to a stable metabolite in plasma incubations and nine metabolites across two in vitro incubation models, eight of them generated by amide-bond cleavage. Chemical stability in a clean buffer is a separate question from proteolytic survival in a biological matrix, so the intact peptide should be confirmed by LC-MS at the end of a long exposure.
- How should lyophilized BPC-157 be stored?
- Tightly closed at −20 °C, protected from light and moisture, and warmed to room temperature in a desiccator before opening. Solutions should be aliquoted and frozen, with freeze–thaw cycles avoided.
Sources & Further Reading
- National Center for Biotechnology Information. PubChem Compound Summary for CID 9941957, BPC 157. PubChem CID 9941957.
- Sikirić P, Petek M, Ručman R, Seiwerth S, Grabarević Ž, Rotkvić I, et al. A new gastric juice peptide, BPC. An overview of the stomach-stress-organoprotection hypothesis and beneficial effects of BPC. Journal of Physiology-Paris 1993;87(5):313–327. doi:10.1016/0928-4257(93)90038-U
- Bódis B, Karádi O, Németh P, Dohoczky C, Kolega M, Mózsik G. Evidence for direct cellular protective effect of PL-10 substances (synthesized parts of body protection compound, BPC) and their specificity to gastric mucosal cells. Life Sciences 1997;61(16):PL243–PL248. doi:10.1016/S0024-3205(97)00744-3
- Tkalčević VI, Čužić S, Brajša K, Mildner B, Bokulić A, Šitum K, et al. Enhancement by PL 14736 of granulation and collagen organization in healing wounds and the potential role of egr-1 expression. European Journal of Pharmacology 2007;570(1–3):212–221. doi:10.1016/j.ejphar.2007.05.072
- Chang CH, Tsai WC, Lin MS, Hsu YH, Pang JHS. The promoting effect of pentadecapeptide BPC 157 on tendon healing involves tendon outgrowth, cell survival, and cell migration. Journal of Applied Physiology 2011;110(3):774–780. doi:10.1152/japplphysiol.00945.2010
- Chang CH, Tsai WC, Hsu YH, Pang JHS. Pentadecapeptide BPC 157 enhances the growth hormone receptor expression in tendon fibroblasts. Molecules 2014;19(11):19066–19077. doi:10.3390/molecules191119066
- Huang T, Gu J, Zhang K, Sun L, Xue X, Zhang C, et al. Body protective compound-157 enhances alkali-burn wound healing in vivo and promotes proliferation, migration, and angiogenesis in vitro. Drug Design, Development and Therapy 2015;9:2485. doi:10.2147/DDDT.S82030
- Hsieh MJ, Liu HT, Wang CN, Huang HY, Lin Y, Ko YS, et al. Therapeutic potential of pro-angiogenic BPC157 is associated with VEGFR2 activation and up-regulation. Journal of Molecular Medicine 2017;95(3):323–333. doi:10.1007/s00109-016-1488-y
- Hsieh MJ, Lee CH, Chueh HY, Chang GJ, Huang HY, Lin Y, Pang JHS. Modulatory effects of BPC 157 on vasomotor tone and the activation of Src-Caveolin-1-endothelial nitric oxide synthase pathway. Scientific Reports 2020;10:17078. doi:10.1038/s41598-020-74022-y
- Cox HD, Miller GD, Eichner D. Detection and in vitro metabolism of the confiscated peptides BPC 157 and MGF R23H. Drug Testing and Analysis 2017;9(10):1490–1498. doi:10.1002/dta.2152
- Tian T, Jing J, Li Y, Wang Y, Deng X, Shan Y. Stable isotope labeling-based nontargeted strategy for characterization of the in vitro metabolic profile of a novel doping BPC-157 in doping control by UHPLC-HRMS. Molecules 2023;28(21):7345. doi:10.3390/molecules28217345
- Józwiak M, Bauer M, Kamysz W, Kleczkowska P. Multifunctionality and possible medical application of the BPC 157 peptide: literature and patent review. Pharmaceuticals 2025;18(2):185. doi:10.3390/ph18020185
- Merrifield RB. Solid phase peptide synthesis. I. The synthesis of a tetrapeptide. Journal of the American Chemical Society 1963;85(14):2149–2154. doi:10.1021/ja00897a025
- Carpino LA, Han GY. 9-Fluorenylmethoxycarbonyl amino-protecting group. The Journal of Organic Chemistry 1972;37(22):3404–3409. doi:10.1021/jo00795a005
- Mergler M, Dick F, Sax B, Weiler P, Vorherr T. The aspartimide problem in Fmoc-based SPPS. Part I. Journal of Peptide Science 2003;9(1):36–46. doi:10.1002/psc.430
- Wedemeyer WJ, Welker E, Scheraga HA. Proline cis–trans isomerization and protein folding. Biochemistry 2002;41(50):14637–14644. doi:10.1021/bi020574b
- Adzhubei AA, Sternberg MJE, Makarov AA. Polyproline-II helix in proteins: structure and function. Journal of Molecular Biology 2013;425(12):2100–2132. doi:10.1016/j.jmb.2013.03.018
- Breci LA, Tabb DL, Yates JR, Wysocki VH. Cleavage N-terminal to proline: analysis of a database of peptide tandem mass spectra. Analytical Chemistry 2003;75(9):1963–1971. doi:10.1021/ac026359i
- Mant CT, Chen Y, Yan Z, Popa TV, Kovacs JM, Mills JB, et al. HPLC analysis and purification of peptides. Methods in Molecular Biology 2007;386:3–55. doi:10.1007/978-1-59745-430-8_1
- Cornish J, Callon KE, Lin CQ, Xiao CL, Mulvey TB, Cooper GJS, Reid IR. Trifluoroacetate, a contaminant in purified proteins, inhibits proliferation of osteoblasts and chondrocytes. American Journal of Physiology-Endocrinology and Metabolism 1999;277(5):E779–E783. doi:10.1152/ajpendo.1999.277.5.E779
Last reviewed:
In the research library
Everything the library holds on BPC-157, and the methods behind the numbers on its certificate.
- BPC-157 reference entry Identity, calculated properties, the mass spectrometry ions to expect and analytical notes, from the structure.
- Check a certificate against this sequence Paste the masses from a spectrum or a certificate; the mass-match tool compares them with what this sequence should give.
- Peptide calculator, with this sequence Formula, average and monoisotopic mass, charge across pH, isoelectric point and absorbance, recalculated as you edit.
- BPC-157 and TB-500 compared Unrelated in sequence and origin. BPC-157 is a linear 15-residue peptide, rich in proline, with free termini. TB-500 is a seven-residue N-acetylated peptide, residues 17–23 of thymosin β4, with a free C-terminal acid. They are compared because the two are often paired in research-material blends, where each must be identified and measured on its own.
- How to read a certificate of analysis What a peptide certificate of analysis should contain, how to check that it belongs to the material in hand, how to read its identity and purity results, and the signs that it deserves a second look.
- HPLC purity analysis of peptides How reversed-phase HPLC measures the chromatographic purity of a peptide, what the figure includes, and what it leaves out.
- Mass spectrometry for peptide identity How mass spectrometry confirms that a peptide is the intended sequence: electrospray and MALDI, working out the expected mass, reading charge states and adducts, sequence confirmation, and the limits of the method.
- Net peptide content and purity: two different numbers Why a peptide that is 99% pure by HPLC can be only 75–85% peptide by weight: what the powder contains, how each part is measured, and how the two figures combine.
- Preparing peptide solutions in the laboratory From a freeze-dried vial to a solution of known concentration: the arithmetic, the solvent, the charge chemistry and the handling, with the errors each step can introduce and the article that covers it.
- Peptide stability and storage How peptides degrade, chemically and physically, why the dry solid lasts far longer than a solution, which sequences are most at risk, and the storage and handling that slow it down.