CJC-1295 (No DAC)
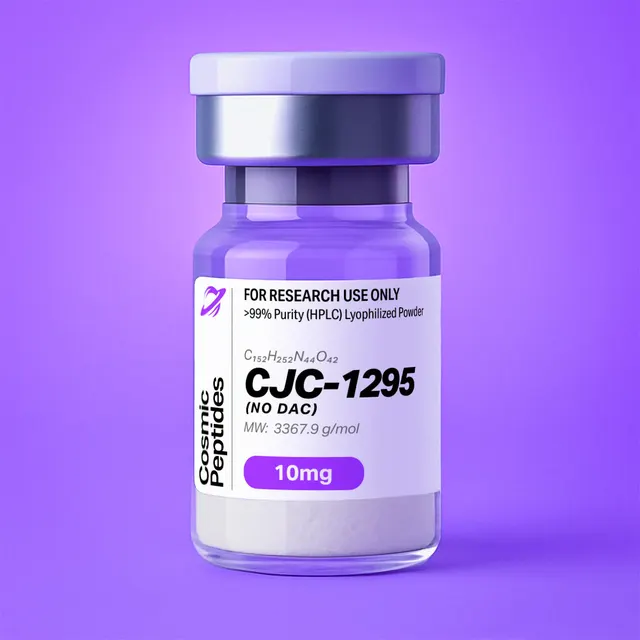
CJC-1295 (No DAC)
Commonly researched with these items
Patent-pending lot tracking: Complete transparency from production to vial.
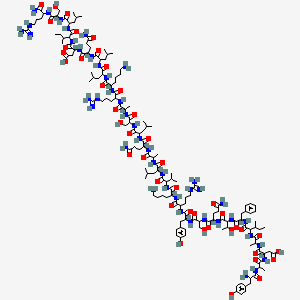
| Molecular Formula | C152H252N44O42 |
|---|---|
| Molecular Weight | 3367.9 g/Mol |
| Sequence | H-Tyr-D-Ala-Asp-Ala-Ile-Phe-Thr-Gln-Ser-Tyr-Arg-Lys-Val-Leu-Ala-Gln-Leu-Ser-Ala-Arg-Lys-Leu-Leu-Gln-Asp-Ile-Leu-Ser-Arg-NH2 |
CJC-1295 (No DAC): Tetrasubstituted GRF(1-29) Amide, a Stabilized Growth Hormone-Releasing Hormone Fragment
Disclaimer
Products described here are supplied for research use only and are not intended for diagnostic, therapeutic, or clinical application. All statements regarding biological activity reflect preclinical and in vitro findings exclusively and have not been evaluated by the U.S. Food and Drug Administration. These materials and related content are provided for educational and investigational purposes only and are intended solely for qualified researchers in laboratory and academic settings.
Key Facts
- Compound class
- Synthetic 29-residue linear peptide amide; analogue of the N-terminal fragment of growth hormone-releasing hormone (GHRH)
- Also known as
- Modified GRF(1-29), [D-Ala2, Gln8, Ala15, Leu27]-GRF(1-29)-NH2, tetrasubstituted GRF(1-29)
- Sequence / structure
H-Tyr-D-Ala-Asp-Ala-Ile-Phe-Thr-Gln-Ser-Tyr-Arg-Lys-Val-Leu-Ala-Gln-Leu-Ser-Ala-Arg-Lys-Leu-Leu-Gln-Asp-Ile-Leu-Ser-Arg-NH₂(one-letter:Y(dA)DAIFTQSYRKVLAQLSARKLLQDILSR-NH₂)- Molecular formula
- C152H252N44O42 (free base)
- Molecular weight
- 3,367.9 g/mol (average); monoisotopic mass 3,365.894 Da
- CAS number
- None reliably assigned to this form; identify it by sequence, formula and PubChem CID 56841945 (stereochemistry defined) or CID 91976842
- Stereochemistry
- All residues L except D-alanine at position 2
- Physical form as supplied
- Lyophilized powder
- Lot traceability
- Every unit is tied to a tracked lot; the lot number, recorded purity and verified quantity of the lot on sale are shown live on this page, with its certificate of analysis.
Molecular Identity and Classification
CJC-1295 (No DAC) is a synthetic 29-amino-acid peptide amide derived from the N-terminal region of growth hormone-releasing hormone (GHRH), the hypothalamic peptide also called growth hormone-releasing factor (GRF). Chemically it is [D-Ala2, Gln8, Ala15, Leu27]-GRF(1-29)-NH2: the first 29 residues of the native sequence, with four single-residue substitutions and a C-terminal carboxamide. In the research literature and in compound databases the same molecule appears as "modified GRF(1-29)" or "tetrasubstituted GRF(1-29)"; PubChem holds it as CID 56841945 (fully stereodefined, systematic name L-tyrosyl-D-alanyl-L-α-aspartyl-…-L-seryl-L-argininamide) and as CID 91976842 ("CJC1295 Without DAC").
Its molecular formula is C152H252N44O42, giving an average molecular weight of 3,367.9 g/mol and a monoisotopic mass of 3,365.894 Da. The composition is Leu ×5, Ala ×4 (one of them D), Arg ×3, Gln ×3, Ser ×3, Asp ×2, Ile ×2, Lys ×2, Tyr ×2, and one each of Phe, Thr and Val. That gives five basic side chains (three arginines, two lysines), two acidic side chains (both aspartate; there is no glutamate), three aromatic residues (two tyrosines and a phenylalanine), and no cysteine, methionine, histidine, proline or tryptophan. The absence of sulfur is itself a useful analytical marker, because the native fragment contains one methionine.
The name deserves explanation because it causes real confusion. "CJC-1295" was introduced for a GRF(1-29) analogue carrying a DAC, the developer's term for an albumin-binding construct: an extra C-terminal lysine whose ε-amino group carries a 3-maleimidopropionyl group, designed to react with the free thiol of albumin to give a covalent conjugate (Jetté and colleagues, 2005). The compound supplied here is the tetrasubstituted peptide without the added lysine and linker, which is why it is labelled "No DAC". The two are different molecules: the DAC form (PubChem CID 91971820) is C165H269N47O46, 3,647.2 g/mol, about 279 Da heavier. Database records for the two names are also cross-contaminated: CAS numbers circulating for "CJC-1295" (for example 863288-34-0 and 446262-90-4) appear in PubChem records alongside the DAC conjugate's name, so neither is a dependable identifier for the No DAC peptide. A researcher comparing data across studies should confirm the form by sequence and mass rather than by name or CAS number.
GHRH itself was isolated and sequenced in 1982 by two groups working independently (Guillemin and colleagues; Rivier and colleagues), both from tumour tissue that over-produced the peptide. The full-length peptide has 44 residues and an amidated C-terminus, but structure–activity work soon showed that the N-terminal 29 residues, amidated, retain high activity at the receptor in cell-based assays. GRF(1-29)-NH2 therefore became the template for a long series of analogues in which individual residues were replaced to address specific chemical weaknesses. CJC-1295 (No DAC) combines four of those replacements in one molecule.
Structure and Chemical Features
Each of the four substitutions addresses a defined chemical liability of the native GRF(1-29) sequence (Tyr-Ala-Asp-Ala-Ile-Phe-Thr-Asn-Ser-Tyr-Arg-Lys-Val-Leu-Gly-Gln-Leu-Ser-Ala-Arg-Lys-Leu-Leu-Gln-Asp-Ile-Met-Ser-Arg-NH2). Understanding them explains most of the compound's analytical and handling behaviour.
| Position | Native residue | Replacement | Monoisotopic mass change | Chemical rationale |
|---|---|---|---|---|
| 2 | L-Ala | D-Ala | 0 Da (stereoisomer) | The Tyr1-Ala2 N-terminus is a substrate motif for dipeptidyl peptidase-4 (DPP-4), which removes N-terminal dipeptides with Pro or Ala at position 2. A D-residue at position 2 is not accepted by the enzyme. |
| 8 | Asn | Gln | +14.016 Da (CH2) | Asn8-Ser9 is a fast-deamidating motif: asparagine followed by a small residue cyclizes to a succinimide that hydrolyses to aspartate and isoaspartate. Glutamine deamidates far more slowly. |
| 15 | Gly | Ala | +14.016 Da (CH2) | Glycine has the lowest α-helix propensity of the proteinogenic amino acids after proline; alanine has the highest. The substitution favours the helical conformation of the central segment. |
| 27 | Met | Leu | −17.956 Da (CH2 − S) | The thioether of methionine oxidizes readily to the sulfoxide. Leucine is a close, non-oxidizable replacement of similar size and hydrophobicity. |
Position 2: resistance to dipeptidyl peptidase-4. Frohman and colleagues showed in 1986 that GHRH incubated in plasma in vitro is rapidly converted to GRF(3-44), a product they described as biologically inactive, by cleavage of the Ala2–Asp3 bond. The enzyme responsible, DPP-4, is a serine protease whose S1 pocket accepts the L-configured side chain of proline or alanine at the penultimate position. Inverting the stereochemistry at position 2 places the methyl side chain where the pocket cannot accommodate it, so the N-terminal dipeptide is not removed. This is the single change with the largest effect on the peptide's integrity in serum-containing media.
Position 8: avoiding deamidation. Deamidation of asparagine proceeds by attack of the following backbone nitrogen on the side-chain carboxamide, forming a five-membered succinimide that hydrolyses to a mixture of aspartyl and isoaspartyl peptides, typically in a ratio near 1:3, with some racemization at the α-carbon (Geiger and Clarke, 1987). The rate depends strongly on the following residue: Asn-Gly is fastest, and Asn-Ser, the motif in native GRF(1-29), is among the next fastest. In a stored peptide this produces impurities with a mass increase of only 0.984 Da that elute close to the parent peak. Glutamine would have to form a less favourable six-membered glutarimide ring and deamidates orders of magnitude more slowly.
Position 15: stabilizing the helix. Structural studies of GHRH analogues, and the cryo-electron microscopy structure of the GHRH receptor bound to its peptide (Zhou and colleagues, 2020), show the peptide adopting a continuous α-helix through most of its length when bound. On the experimental helix propensity scale of Pace and Scholtz, glycine costs 1.0 kcal/mol more than alanine to place in a helix, which is a substantial effect for a single residue in the middle of the chain.
Position 27: removing an oxidation site. Methionine is among the most easily oxidized residues in peptides; its thioether reacts with dissolved oxygen, peroxides and metal-catalysed radicals to form methionine sulfoxide (+15.995 Da), and further to the sulfone (+31.990 Da). Vogt reviewed the chemistry of this modification in 1995. Leucine has nearly the same side-chain volume and hydrophobicity but no sulfur, so the analogue cannot form these oxidation products.
Charge and Conformation
With five basic side chains, two aspartates, a free N-terminal amine and an amidated C-terminus, the peptide carries a net charge of about +4 at pH 7. Using standard side-chain pKa values (N-terminus 9.0, Lys 10.5, Arg 12.5, Asp 3.9, Tyr 10.1), the calculated isoelectric point is about 10.8; the exact figure depends on the pKa set used, but every common set places it above 10. In the helical conformation, hydrophobic residues spaced three or four positions apart (for example Phe6, Val13, Leu17, Leu22 and Ile26) line up along the helix, giving the molecule a partly amphipathic character. In aqueous buffer without a binding partner, GRF(1-29) analogues are largely disordered; helix formation is promoted by membrane-mimetic solvents such as 2,2,2-trifluoroethanol and by binding to the receptor. Circular dichroism in buffer and in buffer–trifluoroethanol mixtures, read at the 208 and 222 nm minima characteristic of α-helix, is the standard way to compare the helical content of GHRH analogues.
Synthesis and Manufacturing Chemistry
CJC-1295 (No DAC) is produced by Fmoc solid-phase peptide synthesis, the approach built on Merrifield's 1963 solid-phase method and Carpino and Han's 9-fluorenylmethoxycarbonyl protecting group. Because the C-terminus is a carboxamide, the chain is assembled on an amide-generating resin such as Rink amide, starting from arginine-29 and finishing with tyrosine-1.
Side chains are protected with acid-labile groups: Pbf (2,2,4,6,7-pentamethyldihydrobenzofuran-5-sulfonyl) on arginine, Boc on lysine, tert-butyl esters on aspartic acid, tert-butyl ethers on serine, threonine and tyrosine, and trityl on glutamine. The D-alanine at position 2 is introduced as Fmoc-D-Ala-OH. At 29 residues the sequence is long enough that aggregation of the growing chain on the resin can slow couplings, particularly through the hydrophobic Leu22-Leu-Gln-Asp-Ile-Leu27 stretch near the C-terminus, which is assembled early; double couplings, elevated temperature, or pseudoproline and backbone-protected building blocks at Ser or Thr positions are common solutions. Three arginines each carrying a bulky Pbf group also make arginine couplings among the slowest in the synthesis.
Two side reactions deserve attention in this sequence. First, aspartic acid residues can cyclize to aspartimide under the basic conditions of repeated Fmoc removal, and the aspartimide then reopens to α- and β-aspartyl peptides and piperidides. The tendency depends on the residue after Asp, being greatest for Asp-Gly and lower for bulkier neighbours (Mergler and colleagues, 2003): of the two junctions here, Asp3-Ala4 is the more susceptible, while Asp25-Ile26 is hindered by the β-branched isoleucine. Additives such as Oxyma or formic acid in the deprotection solution, or bulkier aspartate esters, reduce it. Second, racemization must be controlled at every residue, and the intended D-configuration at position 2 makes stereochemical checking essential: the sequence contains four alanines (positions 2, 4, 15 and 19), so chiral amino-acid analysis after hydrolysis should show D-Ala and L-Ala in a 1:3 ratio, with all other residues L.
Final cleavage with trifluoroacetic acid and scavengers (water, triisopropylsilane) removes the side-chain protecting groups and releases the peptide amide from the resin. Purification by preparative reversed-phase HPLC follows, and the purified fractions are lyophilized. Because trifluoroacetic acid is present throughout, the peptide is commonly isolated as a trifluoroacetate salt, with up to one counterion for each protonated basic group (six: the N-terminal amine, two lysines and three arginines); an ion-exchange step can convert it to the acetate.
Analytical Characterization
Reversed-phase HPLC. Purity is determined on C18 columns with water–acetonitrile gradients containing 0.1% trifluoroacetic acid, with UV detection at 214–220 nm, where the peptide bond absorbs. The peptide is moderately hydrophobic for its size and elutes in the middle of a typical 5–65% acetonitrile gradient. The critical impurities to resolve are deletion sequences (one residue missing) from incomplete couplings, aspartimide-derived and isoaspartyl variants, and the all-L diastereomer (L-Ala2); the last has exactly the same mass and can be distinguished only by chromatography or chiral amino-acid analysis. Shallow gradients (0.25–0.5% acetonitrile per minute) through the elution window improve resolution of these closely related species. Mant and colleagues' methods review is a practical guide to choosing the ion-pairing agent and gradient slope for peptides of this size.
Mass spectrometry. Electrospray ionization produces a series of multiply charged ions, because the six basic sites protonate readily. For the monoisotopic mass of 3,365.894 Da, the expected ions are [M+3H]3+ at m/z 1,122.97, [M+4H]4+ at 842.48, [M+5H]5+ at 674.19 and [M+6H]6+ at 561.99. At this size the monoisotopic peak is not the tallest in each cluster: the calculated isotope pattern has the 13C1 peak (M+1) as the most abundant, M+2 at about 97% of it and the monoisotopic peak at about 54%. Software that picks the tallest peak as "monoisotopic" will therefore report a mass about 1 Da high. Deconvolution of the charge-state envelope gives the neutral mass; at low resolution the average mass, 3,367.9 Da, is the appropriate comparison.
Diagnostic mass shifts. Common modifications are recognized by their exact mass differences: +0.984 Da for deamidation of a glutamine; −18.011 Da for an aspartimide (loss of water); +113.993 Da for a non-covalent trifluoroacetic acid adduct; −71.037 Da or −156.101 Da for deletion of an alanine or arginine; and +10.075 Da relative to native GRF(1-29)-NH2, which is the net effect of the four substitutions and is a quick check that the correct analogue, rather than the native fragment, is present. Because the molecule has no methionine, a +15.995 Da species should be absent; its appearance would point to a mix-up with a methionine-containing analogue rather than oxidation of this peptide.
Sequence confirmation. Tandem MS of the 4+ or 5+ precursor by collision-induced dissociation gives b- and y-ion series. The arginine at the C-terminus produces a strong y-series, and the Arg11, Lys12, Arg20 and Lys21 positions provide charge-retaining fragments across the middle of the chain. Tandem MS confirms the order of residues but not the D-configuration at position 2, which needs chiral analysis or comparison with a reference standard.
Quantity and content. The two tyrosines give a calculated molar absorptivity at 280 nm of about 2,980 M−1cm−1 (1,490 M−1cm−1 per tyrosine; Gill and von Hippel, 1989; Pace and colleagues, 1995), equivalent to an absorbance of about 0.88 for a 1 mg/mL solution of the free base in a 1 cm cell. This allows approximate concentration measurements of stock solutions, although phenylalanine contributes little at 280 nm and light scattering from aggregates can inflate readings. For exact quantities, amino-acid analysis after acid hydrolysis is the reference method. HPLC purity and peptide content are different measures: a sample with high chromatographic purity still contains counterions and water, which can account for 10–20% of the weighed mass (see the worked calculations below).
Physicochemical Properties
| Property | Value | Notes |
|---|---|---|
| Residues | 29 | C-terminal carboxamide; D-Ala at position 2 |
| Molecular formula | C152H252N44O42 | Free base, without counterions; contains no sulfur |
| Average molecular weight | 3,367.9 g/mol | PubChem; agrees with calculation from the sequence |
| Monoisotopic mass | 3,365.894 Da | PubChem 3,365.8935782 Da |
| Principal ESI ions | m/z 1,122.97 (3+), 842.48 (4+), 674.19 (5+), 561.99 (6+) | Protonated, monoisotopic |
| Most abundant isotopologue | M+1 (M+2 at ~97%, M at ~54%) | Calculated from natural isotope abundances |
| Basic / acidic residues | Arg ×3, Lys ×2 / Asp ×2 | No glutamate or histidine |
| Net charge at pH 7 | about +4 | Including the free N-terminal amine |
| Isoelectric point | about 10.8 (calculated) | Depends on the pKa set; above 10 for all common sets |
| Aromatic residues | Tyr ×2, Phe ×1 | No tryptophan |
| ε280 | about 2,980 M−1cm−1 | A280 about 0.88 for 1 mg/mL, 1 cm |
| Computed XLogP3 | −10.7 | PubChem; highly polar overall despite the hydrophobic residues |
| Hydrogen-bond donors / acceptors | 52 / 48 | PubChem computed |
| Topological polar surface area | 1,450 Å2 | PubChem computed |
| Oxidizable residues | None of Met, Cys or Trp | Met27 replaced by Leu |
| Solubility | Soluble in water and dilute aqueous acid | Basic peptide; dissolves readily at slightly acidic pH |
The physicochemical profile is that of a basic, partly amphipathic peptide. The hydrophobic residues (Ile5, Phe6, Val13, Leu14, Leu17, Leu22, Leu23, Ile26, Leu27) explain the peptide's tendency to adsorb to hydrophobic surfaces and, at high concentration in neutral buffers, to self-associate. Slightly acidic solutions, in which all basic groups are fully protonated and charge repulsion keeps molecules apart, generally give the clearest solutions.
Chemically, the four substitutions remove the three fastest degradation pathways of the native fragment: N-terminal enzymatic cleavage, asparagine deamidation and methionine oxidation. The remaining liabilities in solution are slow deamidation of the three glutamines, aspartate isomerization at Asp3 and Asp25 over long storage, and backbone hydrolysis at extremes of pH.
Research Context
CJC-1295 (No DAC) is used as a tool compound in research on the growth hormone-releasing hormone receptor (GHRHR), a class B G protein-coupled receptor. Mayo cloned the receptor in 1992 and showed that, when expressed heterologously, it responds to GHRH with increased intracellular cyclic AMP, consistent with coupling to adenylyl cyclase through Gs. In 2020, Zhou and colleagues determined the cryo-electron microscopy structure of GHRHR bound to GHRH and the Gs heterotrimer, showing how the peptide's N-terminal region inserts deep into the receptor's transmembrane core while the receptor's extracellular domain engages the peptide's C-terminal helical portion. This two-domain binding mode, shared across class B receptors, explains why the N-terminal residues (including Tyr1 and position 2) dominate receptor activation, whereas the central and C-terminal helix contributes mainly to affinity.
These structural and signalling findings define how the compound is studied in vitro. Typical experimental systems include cell lines engineered to express the receptor (for example HEK293 or CHO cells transfected with GHRHR), in which researchers measure cyclic AMP accumulation with homogeneous time-resolved fluorescence or luminescent biosensor assays, receptor binding by competition with a labelled GHRH analogue, and downstream signalling such as phosphorylation of the transcription factor CREB. Concentration–response curves in these assays give EC50 and maximal response values for direct comparison with the native fragment. Primary pituitary cell cultures are also used, in which growth hormone released into the culture medium is measured by immunoassay as a readout of receptor activation in the native cell type.
Because the analogue differs from native GRF(1-29)-NH2 at four defined positions, it is useful in comparative studies that separate potency at the receptor from chemical stability. Side-by-side experiments with the native fragment, with single-substitution analogues, and with the DAC-conjugated form help attribute observed differences to receptor pharmacology, to resistance to DPP-4 in serum-containing media, or to albumin binding. Stability studies commonly incubate the peptides in culture medium or in serum at 37 °C, stop aliquots at set times with acid or organic solvent, and follow the intact peptide and its fragments by LC-MS. In such experiments the native fragment shows the appearance of GRF(3-29)-NH2 (loss of Tyr-Ala, −234.100 Da), whereas the D-Ala2 analogue does not, which makes the comparison a clean demonstration of the position-2 design.
Related GHRH-Receptor Research Peptides
Several peptides in the catalogue share the GHRH scaffold or act on the same hormonal axis through a different receptor. Comparing them is a direct way to study how sequence length, terminal modification and residue substitution affect receptor activity and stability.
| Peptide | Structure | Formula | Average MW (g/mol) | Monoisotopic (Da) |
|---|---|---|---|---|
| Sermorelin | Native GRF(1-29)-NH2 | C149H246N44O42S | 3,357.9 | 3,355.819 (CID 16132413) |
| CJC-1295 (No DAC) | [D-Ala2, Gln8, Ala15, Leu27]-GRF(1-29)-NH2 | C152H252N44O42 | 3,367.9 | 3,365.894 (CID 56841945) |
| CJC-1295 with DAC | The same peptide plus Lys30(ε-3-maleimidopropionyl)-NH2 | C165H269N47O46 | 3,647.2 | 3,645.015 (CID 91971820) |
| Tesamorelin | trans-3-hexenoyl-GHRH(1-44)-NH2 | C221H366N72O67S | 5,136 | 5,132.717 (CID 16137828) |
Sermorelin is the direct parent: the same 29 residues and C-terminal amide, but with L-Ala2, Asn8, Gly15 and Met27. The two differ by only 10.075 Da in monoisotopic mass, so a high-resolution mass measurement or the presence of sulfur (Sermorelin's methionine) cleanly distinguishes them. Tesamorelin takes the opposite approach to N-terminal protection: it keeps the full 44-residue sequence and blocks the N-terminus with an acyl group rather than inverting the stereochemistry at position 2. Ipamorelin is unrelated in structure, a pentapeptide that acts at a different receptor, the growth hormone secretagogue receptor (GHSR1a); it is a useful contrast in cell-based work because its signalling runs through Gq and calcium rather than Gs and cyclic AMP.
Worked Calculations
Mass from the Parent Fragment
The monoisotopic mass of CJC-1295 (No DAC) can be derived from native GRF(1-29)-NH2 (3,355.8187 Da) by adding the effect of each substitution: D-Ala2, 0; Asn→Gln at position 8, +CH2 = +14.0157; Gly→Ala at position 15, +CH2 = +14.0157; Met→Leu at position 27, +CH2 − S = 14.0157 − 31.9721 = −17.9564. The net change is +10.0749 Da, giving 3,365.8936 Da, which matches the PubChem value of 3,365.8935782 Da. The same bookkeeping on the formula, C149H246N44O42S + C3H6 − S, gives C152H252N44O42.
Salt Form, Peptide Content and Molarity
Lyophilized peptides are salts, so the weighed mass is larger than the mass of peptide it contains. Each trifluoroacetate adds 114.02 g/mol (as CF3COOH) and each acetate 60.05 g/mol. The table shows the theoretical peptide fraction for typical salt stoichiometries, before any allowance for water.
| Form | Molar mass (g/mol) | Peptide fraction | Peptide in 1.000 mg weighed |
|---|---|---|---|
| Free base | 3,367.9 | 100% | 1.000 mg (0.297 µmol) |
| · 4 TFA | 3,824.0 | 88.1% | 0.881 mg |
| · 5 TFA | 3,938.1 | 85.5% | 0.855 mg |
| · 6 TFA (all basic sites) | 4,052.1 | 83.1% | 0.831 mg |
| · 6 acetate | 3,728.3 | 90.3% | 0.903 mg |
For molar work: 1.000 mg of free-base peptide is 1.000 / 3,367.9 = 0.297 µmol, so 1.000 mg dissolved to 1.000 mL gives 0.297 mM (297 µM). If the certificate of analysis reports a peptide content of 83%, a 1.000 mg/mL solution of the powder contains 0.83 mg/mL of peptide, or 0.246 mM. A 10 µM working solution is then made by diluting that stock 24.6-fold. Using the free-base molar mass without the content correction overstates the concentration by about 20% for a fully TFA-salted sample.
Laboratory Handling and Storage
Storage of the solid. Keep the lyophilized peptide tightly closed at −20 °C, protected from light and moisture. Allow the vial to reach room temperature in a desiccator before opening, so that atmospheric moisture does not condense on the cold, hygroscopic powder; trifluoroacetate salts are particularly hygroscopic.
Preparing solutions. The peptide dissolves readily in high-purity water or in dilute acetic acid (for example 0.1%), which keeps the basic residues fully protonated and minimizes self-association. Stock solutions of 1 mg/mL (about 0.3 mM) are convenient. For molar concentrations, correct the weighed mass for peptide content rather than assuming the powder is pure peptide. Divide stocks into single-use aliquots and store frozen at −20 °C or −80 °C; avoid repeated freeze–thaw cycles. For cell-based assays, dilute into the assay buffer immediately before use.
Minimizing losses. Peptides of this size and hydrophobicity adsorb to plastic and glass at low concentrations, and losses become significant below about 10 µg/mL. Low-binding polypropylene tubes, and a carrier protein such as bovine serum albumin (0.1%) in assay buffers where the design allows it, reduce losses in dilute working solutions. When the experiment compares the peptide's stability in serum-containing media, the carrier protein should be omitted from the stability arm, or matched across all arms, so that it does not mask differences between analogues.
Monitoring integrity. An LC-MS check of an aged stock for the +0.984 Da (deamidation) and −18.011 Da (aspartimide) species, and an HPLC check for new early- or late-eluting peaks, confirm that a solution is still fit for use. Neutral to mildly basic buffers accelerate both reactions, so stocks are best held at slightly acidic pH and brought to assay pH only on dilution. The lot's certificate of analysis on this page records the analytical results for the material as supplied.
Frequently Asked Research Questions
- What is CJC-1295 (No DAC)?
- It is [D-Ala2, Gln8, Ala15, Leu27]-GRF(1-29)-NH2, a 29-residue analogue of the N-terminal fragment of growth hormone-releasing hormone with four stabilizing substitutions and a C-terminal amide, also called modified GRF(1-29). Its formula is C152H252N44O42 and its molecular weight 3,367.9 g/mol.
- What is the difference between CJC-1295 with DAC and without DAC?
- CJC-1295 with DAC carries an additional C-terminal lysine bearing a 3-maleimidopropionyl group (the DAC), designed to bind albumin covalently through its free thiol. The No DAC form is the tetrasubstituted peptide alone. The DAC form is C165H269N47O46 (3,647.2 g/mol), about 279 Da heavier, so data for one do not transfer to the other.
- Does CJC-1295 (No DAC) have a CAS number?
- No CAS number is reliably assigned to this form. The numbers that circulate under the name "CJC-1295", such as 863288-34-0 and 446262-90-4, appear in PubChem records alongside the DAC conjugate's name. Identify the material by sequence, formula and mass, or by PubChem CID 56841945.
- Why is position 2 a D-amino acid?
- The native Tyr-Ala N-terminus is cleaved by dipeptidyl peptidase-4, producing GRF(3-29), a fragment that lacks activity at the receptor. A D-alanine at position 2 is not accepted by the enzyme, so the peptide stays intact in serum-containing media.
- Why were asparagine 8 and methionine 27 replaced?
- Asn8-Ser9 deamidates rapidly through a succinimide intermediate, and methionine oxidizes to its sulfoxide. Glutamine and leucine are close structural replacements that are far more stable, removing two common sources of impurities on storage.
- What mass should I see by electrospray mass spectrometry?
- The monoisotopic mass is 3,365.894 Da. Expect a charge-state series including [M+3H]3+ at m/z 1,122.97, [M+4H]4+ at 842.48, [M+5H]5+ at 674.19 and [M+6H]6+ at 561.99. In each isotope cluster the tallest peak is M+1, not the monoisotopic peak.
- How can I tell it apart from Sermorelin analytically?
- Sermorelin (native GRF(1-29)-NH2) is 10.075 Da lighter in monoisotopic mass (3,355.819 Da) and contains sulfur from Met27. High-resolution MS separates them easily; at the 4+ charge state the monoisotopic ions are about 2.5 m/z units apart.
- Which receptor does it act on in cell-based assays?
- The growth hormone-releasing hormone receptor (GHRHR), a class B G protein-coupled receptor that raises cyclic AMP through Gs. Its structure bound to GHRH and Gs was solved by cryo-electron microscopy in 2020.
- How is its activity measured in vitro?
- Commonly by cyclic AMP accumulation in cells expressing GHRHR, by competition binding with a labelled GHRH analogue, by CREB phosphorylation, and by growth hormone released into the medium of primary pituitary cell cultures, measured by immunoassay.
- What solvent should I use to dissolve it?
- High-purity water or dilute acetic acid (about 0.1%). The peptide is basic (calculated pI about 10.8), and slightly acidic conditions keep it fully protonated and reduce self-association.
- How do I calculate the molar concentration of a solution?
- Divide the mass of peptide (weighed mass × peptide content from the certificate of analysis) by 3,367.9 g/mol. For example, 1.000 mg/mL of powder with 83% peptide content is 0.83 mg/mL of peptide, or 0.246 mM.
- How should the lyophilized peptide be stored?
- At −20 °C, tightly closed and protected from light and moisture, warming the vial to room temperature in a desiccator before opening. Solutions are best aliquoted and frozen at −20 °C or −80 °C.
Sources & Further Reading
- Guillemin R, Brazeau P, Böhlen P, Esch F, Ling N, Wehrenberg WB. Growth hormone-releasing factor from a human pancreatic tumor that caused acromegaly. Science 1982;218(4572):585–587. doi:10.1126/science.6812220
- Rivier J, Spiess J, Thorner M, Vale W. Characterization of a growth hormone-releasing factor from a human pancreatic islet tumour. Nature 1982;300(5889):276–278. doi:10.1038/300276a0
- Frohman LA, Downs TR, Williams TC, Heimer EP, Pan YC, Felix AM. Rapid enzymatic degradation of growth hormone-releasing hormone by plasma in vitro and in vivo to a biologically inactive product cleaved at the NH2 terminus. Journal of Clinical Investigation 1986;78(4):906–913. doi:10.1172/JCI112679
- Jetté L, Léger R, Thibaudeau K, et al. Human growth hormone-releasing factor (hGRF)1–29-albumin bioconjugates activate the GRF receptor on the anterior pituitary in rats: identification of CJC-1295 as a long-lasting GRF analog. Endocrinology 2005;146(7):3052–3058. doi:10.1210/en.2004-1286
- Mayo KE. Molecular cloning and expression of a pituitary-specific receptor for growth hormone-releasing hormone. Molecular Endocrinology 1992;6(10):1734–1744. doi:10.1210/mend.6.10.1333056
- Zhou F, Zhang H, Cong Z, et al. Structural basis for activation of the growth hormone-releasing hormone receptor. Nature Communications 2020;11:5205. doi:10.1038/s41467-020-18945-0
- Geiger T, Clarke S. Deamidation, isomerization, and racemization at asparaginyl and aspartyl residues in peptides. Succinimide-linked reactions that contribute to protein degradation. Journal of Biological Chemistry 1987;262(2):785–794. doi:10.1016/S0021-9258(19)75855-4
- Pace CN, Scholtz JM. A helix propensity scale based on experimental studies of peptides and proteins. Biophysical Journal 1998;75(1):422–427. doi:10.1016/S0006-3495(98)77529-0
- Vogt W. Oxidation of methionyl residues in proteins: tools, targets, and reversal. Free Radical Biology and Medicine 1995;18(1):93–105. doi:10.1016/0891-5849(94)00158-G
- Merrifield RB. Solid phase peptide synthesis. I. The synthesis of a tetrapeptide. Journal of the American Chemical Society 1963;85(14):2149–2154. doi:10.1021/ja00897a025
- Carpino LA, Han GY. 9-Fluorenylmethoxycarbonyl amino-protecting group. The Journal of Organic Chemistry 1972;37(22):3404–3409. doi:10.1021/jo00795a005
- Mergler M, Dick F, Sax B, Weiler P, Vorherr T. The aspartimide problem in Fmoc-based SPPS. Part I. Journal of Peptide Science 2003;9(1):36–46. doi:10.1002/psc.430
- Mant CT, Chen Y, Yan Z, et al. HPLC analysis and purification of peptides. Methods in Molecular Biology 2007;386:3–55. doi:10.1007/978-1-59745-430-8_1
- Gill SC, von Hippel PH. Calculation of protein extinction coefficients from amino acid sequence data. Analytical Biochemistry 1989;182(2):319–326. doi:10.1016/0003-2697(89)90602-7
- Pace CN, Vajdos F, Fee L, Grimsley G, Gray T. How to measure and predict the molar absorption coefficient of a protein. Protein Science 1995;4(11):2411–2423. doi:10.1002/pro.5560041120
- PubChem Compound Summary, CID 56841945: L-tyrosyl-D-alanyl-L-α-aspartyl-…-L-seryl-L-argininamide (CJC-1295 without DAC, stereodefined). National Center for Biotechnology Information.
- PubChem Compound Summary, CID 91976842: CJC1295 Without DAC. National Center for Biotechnology Information.
- PubChem Compound Summaries, CID 16132413 (Sermorelin), CID 91971820 (CJC-1295 with DAC) and CID 16137828 (Tesamorelin). National Center for Biotechnology Information.
Last reviewed:
In the research library
Everything the library holds on CJC-1295 (no DAC), and the methods behind the numbers on its certificate.
- CJC-1295 (no DAC) reference entry Identity, calculated properties, the mass spectrometry ions to expect and analytical notes, from the structure.
- Check a certificate against this sequence Paste the masses from a spectrum or a certificate; the mass-match tool compares them with what this sequence should give.
- Peptide calculator, with this sequence Formula, average and monoisotopic mass, charge across pH, isoelectric point and absorbance, recalculated as you edit.
- Growth hormone–releasing hormone analogs The family side by side: sequences aligned, each member's relation to the reference peptide, and how analysis tells them apart.
- Sermorelin and CJC-1295 (no DAC) compared Both are 29-residue C-terminal amides built on the first 29 residues of growth hormone–releasing hormone. CJC-1295 without DAC carries four substitutions in that chain; sermorelin is the unmodified sequence.
- How to read a certificate of analysis What a peptide certificate of analysis should contain, how to check that it belongs to the material in hand, how to read its identity and purity results, and the signs that it deserves a second look.
- HPLC purity analysis of peptides How reversed-phase HPLC measures the chromatographic purity of a peptide, what the figure includes, and what it leaves out.
- Mass spectrometry for peptide identity How mass spectrometry confirms that a peptide is the intended sequence: electrospray and MALDI, working out the expected mass, reading charge states and adducts, sequence confirmation, and the limits of the method.
- Net peptide content and purity: two different numbers Why a peptide that is 99% pure by HPLC can be only 75–85% peptide by weight: what the powder contains, how each part is measured, and how the two figures combine.
- Preparing peptide solutions in the laboratory From a freeze-dried vial to a solution of known concentration: the arithmetic, the solvent, the charge chemistry and the handling, with the errors each step can introduce and the article that covers it.
- Peptide stability and storage How peptides degrade, chemically and physically, why the dry solid lasts far longer than a solution, which sequences are most at risk, and the storage and handling that slow it down.