Epitalon
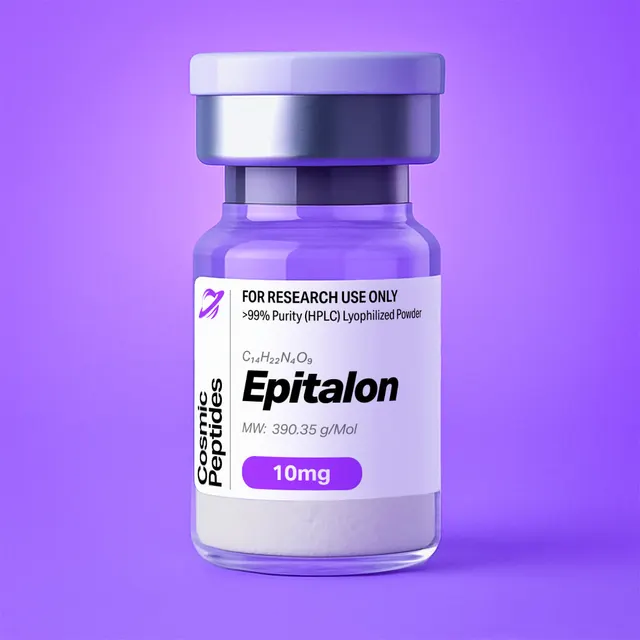
Epitalon
Commonly researched with these items
Patent-pending lot tracking: Complete transparency from production to vial.
| CAS Number | 307297-39-8 |
|---|---|
| Molecular Formula | C14H22N4O9 |
| Molecular Weight | 390.35 g/Mol |
| Purity | 99.8% |
| Lot Number | 26074 |
| Quantity | 10.21mg |
| Sequence | H-Ala-Glu-Asp-Gly-OH |
Epitalon (Ala-Glu-Asp-Gly): An Acidic Synthetic Tetrapeptide Used in Telomerase and Chromatin Research
Disclaimer
Products described here are supplied for research use only and are not intended for diagnostic, therapeutic, or clinical application. All statements regarding biological activity reflect preclinical and in vitro findings exclusively and have not been evaluated by the U.S. Food and Drug Administration. These materials and related content are provided for educational and investigational purposes only and are intended solely for qualified researchers in laboratory and academic settings.
Key Facts
- Compound class
- Linear synthetic tetrapeptide; acidic oligopeptide carrying three carboxylic acid groups and one amine
- Sequence / structure
H-Ala-Glu-Asp-Gly-OH(one-letter code: AEDG), L-alanyl-L-α-glutamyl-L-α-aspartyl-glycine, all chiral residues in the L-configuration- Molecular formula
- C14H22N4O9
- Molecular weight
- 390.35 g/mol (average); monoisotopic mass 390.1387 Da
- CAS number
- 307297-39-8
- PubChem CID
- 219042
- Other identifiers
- FDA UNII O65P17785G; ChEBI 230091; synonyms Epithalon, Epithalone, AEDG
- Physical form as supplied
- Lyophilized powder
- Lot traceability
- Every unit is tied to a tracked lot; the lot number, recorded purity and verified quantity of the lot on sale are shown live on this page, with its certificate of analysis.
Molecular Identity and Classification
Epitalon is the tetrapeptide alanyl-glutamyl-aspartyl-glycine, written H-Ala-Glu-Asp-Gly-OH or AEDG; the spellings Epithalon and Epithalone denote the same molecule, and much of the biochemical literature calls it simply "the AEDG peptide". Its systematic IUPAC name, (4S)-4-[[(2S)-2-aminopropanoyl]amino]-5-[[(2S)-3-carboxy-1-(carboxymethylamino)-1-oxopropan-2-yl]amino]-5-oxopentanoic acid, is written from the glutamic acid residue outwards and encodes three stereocentres, all S (L); glycine is achiral.
The molecular formula is C14H22N4O9, the average molecular weight 390.35 g/mol and the monoisotopic mass 390.1387 Da. By mass the molecule is 43.08% carbon, 5.68% hydrogen, 14.35% nitrogen and 36.89% oxygen, an oxygen-rich composition that reflects its three free carboxylic acids. It is registered under CAS number 307297-39-8, as PubChem compound 219042, as FDA Unique Ingredient Identifier O65P17785G and as ChEBI 230091.
Chemically, Epitalon is a short linear oligopeptide and, within that class, one of the strongly acidic minority. Two of its four residues carry side-chain carboxylic acids, and with the C-terminal carboxyl they outnumber the single basic group, the N-terminal amine. The result is a peptide of net charge about −2 at neutral pH and isoelectric point near pH 3, behaving more like a small polycarboxylic acid than like the cationic peptides that dominate much of peptide research. It contains no aromatic, sulfur-containing or basic side chains: no tryptophan or tyrosine absorbance, no oxidizable methionine or cysteine, no lysine or arginine for tryptic cleavage or cation-exchange retention.
The sequence is a designed one rather than a fragment excised from a precursor protein: it was composed from the amino-acid composition of epithalamin, a polypeptide fraction isolated from bovine pineal tissue in the 1970s (see History of the Molecule below). Hence Epitalon is usually discussed alongside short synthetic peptides of the same tradition, such as Lys-Glu-Asp-Gly, Ala-Glu-Asp-Leu and Pinealon (Glu-Asp-Arg), which share an internal Glu-Asp motif.
Structure and Chemical Features
Each residue contributes a distinct feature. Alanine supplies the molecule's only primary amine, its α-amino group, with a methyl side chain that is its sole hydrophobic element. Glutamic acid carries a three-carbon side chain ending in a γ-carboxylic acid, aspartic acid a shorter two-carbon side chain ending in a β-carboxylic acid, and glycine, side chain a hydrogen atom, closes the sequence with the free C-terminal carboxyl and maximal backbone flexibility. Every residue except glycine is chiral; the three peptide bonds are Ala–Glu, Glu–Asp and Asp–Gly.
PubChem's computed descriptors summarize the consequences: 7 hydrogen-bond donors, 10 hydrogen-bond acceptors, 12 rotatable bonds, a topological polar surface area of 225 Å2 and a calculated XLogP3 of −5.5. A membrane-permeable small molecule typically falls below about 140 Å2, so Epitalon is one of the most hydrophilic of the commonly studied short peptides.
Two motifs govern its chemistry. The first is the Asp–Gly junction: glycine has no side chain to hinder the approach, so its backbone nitrogen can attack the side-chain carbonyl of the preceding aspartic acid and close a five-membered succinimide (aspartimide) ring, the most reactive arrangement of its kind in peptide chemistry and the one that shapes both synthesis and solution stability here. The second is side-chain-linked isomerism: glutamic and aspartic acid each have two carboxyl groups, so a peptide of identical mass can be built through the γ-carboxyl of glutamic acid or the β-carboxyl of aspartic acid. Araj and colleagues noted in 2025 that at least one publication presented such a "double-gamma bonded" structure under the Epitalon name: composition and mass alone do not define the molecule.
Charge States and Conformation in Solution
Four groups titrate: the C-terminal carboxyl (pKa roughly 3.1 to 3.6 in short peptides), the aspartic acid side chain (about 3.9), the glutamic acid side chain (about 4.1 to 4.3) and the N-terminal amine (about 7.7 to 8.6 for alanine, by reference set). The calculated isoelectric point then falls between about pH 3.0 and 3.7, with net charge roughly +0.7 to +1 at pH 2, about −1.7 at pH 5 and about −2 at pH 7.0 to 7.4, approaching −3 above pH 9. The table gives one worked set, using mid-range values (C-terminus 3.3, Asp 3.9, Glu 4.2, N-terminal amine 8.0) and the Henderson–Hasselbalch relation for each group.
| pH | Net charge | Practical meaning |
|---|---|---|
| 2.0 | +0.93 | 0.1% TFA mobile phase: nearly fully protonated, best reversed-phase retention |
| 3.0 | +0.49 | Formic acid mobile phase; close to the isoelectric point, lowest solubility |
| 4.0 | −0.78 | Carboxyls titrating; retention changes steeply with small pH shifts |
| 5.0 | −1.77 | Acetate buffer range |
| 7.4 | −2.20 | Culture media and HEPES or phosphate buffers; anion-exchange retention |
| 9.0 | −2.91 | Amine largely neutral; ammonium bicarbonate eluents |
The peptide is too short for regular secondary structure, but it is not a featureless random coil either. Molecular-dynamics simulations of the zwitterion in explicit water, reported by Rogachevskii, Shchegolev and Khavinson in 2006, found the lowest-energy conformers stabilized by two intramolecular salt bridges between the protonated N-terminal amine and the side-chain carboxylates of glutamic and aspartic acid, plus an intramolecular hydrogen bond. Such contacts reduce the conformational freedom of the chain and make the ensemble sensitive to pH and ionic strength, since salt bridges weaken when the amine is deprotonated or when added salt screens the charges.
Synthesis and Manufacturing Chemistry
Epitalon is produced by solid-phase peptide synthesis (SPPS), the approach Merrifield introduced in 1963 with, fittingly, a tetrapeptide. Practice combines the base-labile 9-fluorenylmethoxycarbonyl (Fmoc) group described by Carpino and Han in 1972 on the α-amine with acid-labile tert-butyl esters on the side-chain carboxyls, so the building blocks are Fmoc-Gly-OH, Fmoc-Asp(OtBu)-OH, Fmoc-Glu(OtBu)-OH and Fmoc-Ala-OH. Assembly runs from the C-terminus: glycine is loaded on the resin, then aspartic acid, glutamic acid and alanine are coupled in turn, each after Fmoc removal with base, typically 20% piperidine in dimethylformamide.
The Asp–Gly junction makes this short sequence more demanding than its length suggests. During each piperidine exposure after aspartic acid has been coupled, the deprotonated glycine amide nitrogen can attack the tert-butyl ester of the aspartic acid side chain, expelling tert-butanol and closing an aspartimide ring. Asp–Gly is the sequence most prone to this reaction, and it is the motif Mergler and colleagues chose for their 2003 model hexapeptide H-Val-Lys-Asp-Gly-Tyr-Ile-OH: a bulkier 3-methylpent-3-yl ester on the aspartyl side chain reduced aspartimide formation markedly, and backbone protection of the glycine with a 2-hydroxy-4-methoxybenzyl (Hmb) group together with the tert-butyl ester suppressed it completely. The ring can be reopened by water or piperidine, giving a mixture of the correct α-aspartyl peptide, the isomeric β-aspartyl peptide, their D-aspartyl epimers and piperidide adducts, and since the α- and β-products share a mass and behave similarly on reversed phase, the problem is better avoided than corrected. The countermeasures, reviewed by Subirós-Funosas, El-Faham and Albericio in 2011, are an acidic additive such as HOBt or Oxyma in the piperidine solution, bulkier side-chain esters than tert-butyl, or masking the glycine backbone nitrogen with an Hmb or 2,4-dimethoxybenzyl (Dmb) group, most conveniently by coupling the preformed dipeptide Fmoc-Asp(OtBu)-(Dmb)Gly-OH. Epitalon has one advantage over longer Asp–Gly peptides: only three Fmoc removals follow the aspartic acid coupling, so cumulative base exposure is short.
A second sequence-specific side reaction occurs at the dipeptide stage. When the Fmoc group is removed from resin-bound H-Asp(OtBu)-Gly, the free amine can attack the ester link to the resin and cyclize into the diketopiperazine cyclo(Asp-Gly), cleaving the chain from the support; hindered 2-chlorotrityl chloride resin and prompt coupling of the third residue suppress that loss. A single trifluoroacetic acid (TFA) cleavage with water and triisopropylsilane as scavengers then releases the peptide and removes all tert-butyl groups, and the crude material is precipitated in cold ether, purified by preparative reversed-phase HPLC and lyophilized. Because Epitalon has only one basic group it binds at most about one equivalent of trifluoroacetate, and its acidic character also allows isolation as the free acid or as a partial sodium or ammonium salt; each lot's certificate of analysis states the analytical results for that material.
Analytical Characterization
Epitalon is small enough to be characterized completely, and its acidity shapes every method. Reversed-phase HPLC with UV detection at 210 to 220 nm is the standard purity method: the three peptide bonds are the only significant chromophore, since the molecule has no aromatic residue and essentially no 280 nm absorbance. With an XLogP3 of −5.5 it is weakly retained on conventional C18 phases and elutes close to the void volume; retention improves with an aqueous-stable (polar-embedded or "AQ") C18 column starting at 0 to 2% acetonitrile, an acidic mobile phase (0.1% TFA or formic acid) that protonates the carboxyls, or a more hydrophobic ion-pairing agent, and hydrophilic interaction chromatography (HILIC) is a useful orthogonal method.
Mass spectrometry confirms identity. Positive electrospray gives [M+H]+ at m/z 391.1460; with only one basic site, [M+2H]2+ (196.0766) is weak, while alkali adducts [M+Na]+ (413.1279) and [M+K]+ (429.1018) are common once carboxyls have exchanged with sodium. Negative-mode ESI suits this acidic peptide and gives [M−H]− at 389.1314, and the 13C isotope pattern is an internal check: M+1 should be about 17% of the monoisotopic peak for 14 carbons.
Fragmentation and Isomer Discrimination
Collision-induced dissociation of [M+H]+ cleaves the three amide bonds to give the b- and y-type ions tabulated below, and the mobile-proton framework of Wysocki and colleagues explains their relative intensities. Selective cleavage C-terminal to aspartic acid, driven by the Asp side-chain carboxyl, is pronounced when the ionizing proton is sequestered by arginine; Epitalon has no arginine, lysine or histidine, so the proton of [M+H]+ is mobile and all three amide bonds cleave, giving b2/y2 and b3/y1 pairs rather than one dominant fragment. The small y1 ion (m/z 76.0393) falls below the low-mass cut-off of many ion traps, so on such instruments b3 (m/z 316.1139), b2 and y3 carry the sequence information. Note one isobaric coincidence: y3 (Glu-Asp-Gly) has the same m/z, 320.1088, as the protonated des-Ala deletion peptide, so a peak at 320.109 in a full-scan spectrum is either an in-source fragment or an impurity, and only its chromatographic retention tells them apart.
| Species | m/z (calculated) | Notes |
|---|---|---|
| [M+H]+ | 391.1460 | Principal positive-mode ion |
| [M+2H]2+ | 196.0766 | Weak: one basic site only |
| [M+Na]+ / [M+K]+ | 413.1279 / 429.1018 | Common adducts of an acidic peptide |
| [M−H]− | 389.1314 | Principal negative-mode ion |
| b2 (Ala-Glu) / y2 (Asp-Gly) | 201.0870 / 191.0662 | Cleavage of the Glu–Asp bond |
| b3 (Ala-Glu-Asp) / y1 (Gly) | 316.1139 / 76.0393 | Cleavage C-terminal to Asp, expected to be favoured |
| y3 (Glu-Asp-Gly) | 320.1088 | Distinguishes AEDG from the sequence isomer EADG (y3 Ala-Asp-Gly, 262.1034); both share b2 201.0870 |
| Aspartimide (succinimide) form, [M−H2O+H]+ | 373.1354 | −18.0106 Da; synthesis or storage by-product |
| Aspartimide piperidide, [M+H]+ | 458.2245 | +67.0786 Da relative to the peptide; synthesis by-product |
| Deletion peptides, [M+H]+ | des-Ala 320.1088; des-Glu 262.1034; des-Asp 276.1190; des-Gly 334.1245 | Incomplete couplings |
Mass alone cannot distinguish Epitalon from three classes of isomer, all C14H22N4O9: the β-aspartyl (isoaspartyl) isomer formed when an aspartimide reopens on the wrong side, which elutes slightly apart from the α-form; any side-chain-linked isomer built through the γ-carboxyl of glutamic acid; and a sequence isomer such as Glu-Ala-Asp-Gly (EADG), which gives a different y3 ion (262.1034 instead of 320.1088). A thermal stress test is no shortcut here: an N-terminal glutamic acid would cyclize to pyroglutamate with loss of 18.0106 Da, but heating Epitalon in solution also drives succinimide formation at Asp–Gly with exactly the same mass loss, so the two −18 Da products can only be told apart by MS/MS (pyroglutamate shifts the b ions, the succinimide the y2 and y3 ions).
For quantitative work, purity and peptide content must be kept apart: HPLC purity is the fraction of UV-absorbing material that is the target peptide, while peptide content is the fraction of the weighed powder that is peptide rather than counterion, water or salt. A mono-trifluoroacetate salt has a formula weight of 390.35 + 114.02 = 504.37 g/mol, so even perfectly dry, 100% pure material of that form is 77.4% peptide by weight; a monosodium salt (C14H21N4NaO9) weighs 412.33 g/mol. Amino-acid analysis after hydrolysis (expected molar ratio Ala : Glx : Asx : Gly of 1 : 1 : 1 : 1) or quantitative NMR gives peptide content, ion chromatography the counterion, Karl Fischer titration the water, and chiral analysis the D-aspartic acid that signals aspartimide-mediated epimerization.
NMR spectroscopy fingerprints so small a molecule completely: in D2O the 1H spectrum shows the alanine methyl doublet near 1.4 to 1.5 ppm, the glutamic acid β- and γ-methylene multiplets between about 1.9 and 2.5 ppm, the aspartic acid β-methylene pair near 2.7 to 2.9 ppm, the glycine α-methylene near 3.8 to 4.0 ppm and three α-CH resonances between 4.0 and 4.7 ppm. Because these shifts move with pH, spectra belong at a stated pD, and a β-aspartyl isomer shows altered aspartyl shifts.
Physicochemical Properties
| Property | Value | Notes |
|---|---|---|
| Molecular formula | C14H22N4O9 | Free peptide, without counterions |
| Average molecular weight | 390.35 g/mol | PubChem CID 219042 |
| Monoisotopic mass | 390.1387 Da | For high-resolution MS |
| Elemental composition | C 43.08%, H 5.68%, N 14.35%, O 36.89% | Calculated from the formula |
| Titratable groups | 3 carboxyl, 1 amine | C-terminus, Asp, Glu; N-terminal Ala |
| Isoelectric point | about 3.0–3.7 (calculated) | Range reflects different pKa reference sets |
| Net charge at pH 7.4 | about −2 | Strongly anionic |
| XLogP3 | −5.5 | Computed; extremely hydrophilic |
| Topological polar surface area | 225 Å2 | Computed |
| Hydrogen-bond donors / acceptors | 7 / 10 | Computed |
| Rotatable bonds | 12 | Computed |
| UV absorbance | Peptide bonds only (about 214 nm) | No aromatic residues; no 280 nm signal |
| Oxidation-sensitive residues | None | No Met, Cys or Trp |
| Chemically labile motif | Asp–Gly | Succinimide formation and isoaspartate |
| Amount of substance per 10 mg / 50 mg | 25.6 µmol / 128.1 µmol | Assuming 100% peptide content |
The profile follows directly from the composition. Epitalon dissolves readily in water and in neutral buffers, where its three ionized carboxylates make it highly charged and strongly hydrated; solubility is lowest near the isoelectric point, around pH 3, which matters in acidic mobile phases at high loading. The lyophilized solid is hygroscopic and takes up water that adds to the weighed mass, and the strongly negative partition coefficient makes passive diffusion across lipid bilayers negligible, so any entry into cells must involve transporters, endocytosis or another carrier-mediated route.
One consequence is easy to overlook: an acidic free peptide acidifies the solution it is dissolved in. Bringing Epitalon to pH 7.4 releases roughly two protons per molecule, so a 10 mM solution delivers of the order of 20 mM acid, beyond the capacity of a phosphate-buffered saline containing about 10 mM phosphate. Concentrated stocks should be checked with a pH meter and adjusted if necessary; at low-micromolar working concentrations the effect is negligible.
Research Context
The in vitro literature falls into three lines of work: telomerase and telomere length in cultured cells; entry into cells and nuclei, with binding to nucleic acids and histones; and gene expression in cultured stem-cell populations. One question unites them: how can a short, polar, anionic tetrapeptide alter gene expression inside a cell, and what does it bind? No receptor has been identified, and Araj and colleagues note in 2025 that physico-chemical and structural studies remain few beside the volume of biological reports.
Telomerase and Telomere Length in Cultured Cells
Telomerase is the ribonucleoprotein reverse transcriptase that adds TTAGGG repeats to chromosome ends; Greider and Blackburn identified the activity in Tetrahymena extracts in 1985. It comprises a catalytic subunit, TERT (gene hTERT), and an RNA template. Most cultured somatic cell strains express little or none, whereas most immortalized and cancer-derived lines do, as Kim and colleagues showed in 1994 with the PCR-based telomeric repeat amplification assay (TRAP) they introduced; telomerase-negative strains are therefore the informative system for asking whether a compound induces the enzyme.
In 2003, Khavinson, Bondarev and Butyugov reported that adding Epitalon to telomerase-negative fetal fibroblast cultures induced expression of the catalytic subunit, measurable telomerase activity and telomere elongation; that report set the question later work has tried to quantify.
A 2025 study by Al-Dulaimi, Thomas, Matta and Roberts gave the most detailed quantitative data so far. Two telomerase-positive breast cancer lines (21NT, BT474) were exposed to 0.1, 0.2, 0.5 and 1.0 µg/mL Epitalon (about 0.26 to 2.6 µM) daily for 4 days, and a normal fibroblast strain (IBR.3) and mammary epithelial cells (HMEC) to 1.0 µg/mL daily for 3 weeks, with four read-outs: telomere length by quantitative PCR against a single-copy gene, hTERT mRNA by RT-qPCR, telomerase activity by a qPCR-based TRAP assay against a TERT-overexpressing line, and the telomerase-independent alternative lengthening of telomeres (ALT) pathway by C-circle assay with PML-body immunofluorescence.
The results separated two mechanisms. In the fibroblast and epithelial cultures the 3-week exposure raised telomere length, hTERT mRNA and telomerase activity (about fourfold in IBR.3 and 26-fold in HMEC against unexposed controls), while a 4-day exposure of IBR.3 changed nothing. In both cancer lines telomere length and hTERT mRNA also rose while telomerase activity did not; instead C-circle levels increased about tenfold in 21NT and threefold in BT474, with more PML bodies, indicating ALT activation, which the normal cells showed little (HMEC) or not at all (IBR.3). The authors offered binding to linker histone H1 variants as a hypothesis for the ALT response, and noted the limits of a two-dimensional culture study and of qPCR telomere measurement; a correction to the article is published (doi:10.1007/s10522-025-10326-8). Method points follow for comparable work: qPCR telomere length (Cawthon, 2002) averages over all chromosome ends, so terminal restriction fragment analysis adds distribution data; TRAP needs a heat-inactivated negative control and a telomerase-positive reference; and the C-circle assay of Henson and colleagues (2009), which quantifies extrachromosomal partly single-stranded telomeric circles as a specific ALT marker, needs a phi29-polymerase-free control and an ALT-positive reference line (the 2025 study expressed C-circle levels relative to U2OS cells).
Cellular Uptake and Interaction With DNA and Histones
Fedoreyeva and colleagues addressed the uptake question in 2011. They incubated HeLa cells with fluorescein isothiocyanate (FITC)-labelled Epitalon, Pinealon (Glu-Asp-Arg) and Lys-Glu-Asp-Gly and saw fluorescence in cytoplasm, nucleus and nucleolus. In cell-free experiments the unlabelled peptides quenched the fluorescence of 5,6-carboxyfluorescein-labelled deoxyribooligonucleotides to different extents, expressed as Stern–Volmer constants, and altered the fluorescence of DNA–ethidium bromide complexes; Epitalon appeared to prefer oligonucleotides containing CNG and specifically CAG sequences, targets of cytosine methylation, with binding sensitive to the methylation state. In 2013 the same group extended the work to short peptides binding FITC-labelled wheat histones. Two caveats attach: the label roughly doubles the mass of a 390 Da peptide, so uptake of the conjugate need not reflect uptake of the free peptide, and quenching constants depend on ionic strength.
Gene Expression in Stem-Cell Cultures
In 2020, Khavinson and colleagues reported that Epitalon raised the mRNA levels of the neuronal differentiation markers Nestin, GAP43, β-tubulin III and doublecortin by 1.6- to 1.8-fold in cultured gingival mesenchymal stem cells, with matching increases in the proteins. Molecular docking in the same paper favoured binding to the linker histone variants H1/6 and H1/3 at sites that themselves contact DNA, while the core histones H2b, H3 and H4 offered no suitable site. That is the prediction the 2025 telomere study invoked for ALT induction, which makes histone H1 binding a concrete hypothesis for isothermal titration calorimetry, NMR titration or surface plasmon resonance, none yet reported for this peptide.
The cell-culture designs cited here use sub-micromolar to low-micromolar concentrations (0.26 to 2.6 µM in the 2025 telomere study), repeated additions with daily medium changes over days to weeks, and read-outs by RT-qPCR, immunoblotting, immunofluorescence and enzyme-activity assays. Because the peptide is acidic, the vehicle should be matched for pH and counterion, and its persistence in conditioned medium checked by LC-MS.
History of the Molecule
The chemistry of Epitalon begins with an extract. In 1973 the name epithalamin first appeared in widely accessible literature for a polypeptide fraction obtained from bovine pineal tissue, whose early study was led mainly by V. K. Khavinson's group. Like other tissue extracts of its time it was a heterogeneous mixture defined by its source and preparation rather than by a structure, and the programme that followed set out to reduce it to one defined synthetic molecule.
The approach was compositional: the amino-acid composition of the extract guided the design of short peptides, and Ala-Glu-Asp-Gly emerged as the synthetic representative of the fraction, its synthesis patented in 2000. For years the tetrapeptide itself had not been shown to occur in the natural material; according to the 2025 review by Araj and colleagues it was first detected directly in a pineal polypeptide complex preparation in 2017, by the same high-resolution LC-MS that underpins identity testing today.
Related Short Peptides
Epitalon belongs to a family of short synthetic peptides that share a Glu-Asp core flanked by different residues; comparing their chemistry clarifies what is specific to AEDG. The table lists calculated values for the free peptides.
| Peptide | Formula | Average MW (g/mol) | [M+H]+ (m/z) | Charge character at pH 7 |
|---|---|---|---|---|
| Epitalon, Ala-Glu-Asp-Gly (AEDG) | C14H22N4O9 | 390.35 | 391.1460 | About −2; contains Asp–Gly |
| Lys-Glu-Asp-Gly (KEDG) | C17H29N5O9 | 447.44 | 448.2038 | About −1; an added lysine amine |
| Ala-Glu-Asp-Leu (AEDL) | C18H30N4O9 | 446.46 | 447.2086 | About −2; Leu adds hydrophobicity |
| Pinealon, Glu-Asp-Arg (EDR) | C15H26N6O8 | 418.41 | 419.1885 | About 0; Arg balances two acids |
Three comparisons are informative. Lysine in place of the N-terminal alanine (KEDG) adds a side-chain amine and raises the net charge by one unit, changing the isoelectric point and the ion-exchange behaviour while leaving the Asp–Gly liability untouched; leucine in place of the C-terminal glycine (AEDL) removes that motif altogether, since a bulky residue after aspartic acid hinders succinimide closure; and the near-neutral tripeptide Pinealon shows what one basic residue does, its guanidinium group dominating chromatography and fragmentation alike. For method development the cationic KPV and the copper-coordinating GHK-Cu are useful counterpoints: run all three on one gradient and the retention window is mapped before the method meets unknowns.
Laboratory Handling and Storage
Storage of the solid. Lyophilized Epitalon is best kept tightly closed at −20 °C, protected from light and moisture. Because the powder is hygroscopic, let a vial from the freezer reach room temperature in a desiccator before opening it, so that water does not condense on the cold solid and add to the weighed mass. Weigh with a non-metallic spatula where possible: a carboxylate-rich peptide is a plausible ligand for metal ions, and trace metal pickup is an avoidable source of adduct peaks.
Dissolving, pH and molarity. Epitalon dissolves readily in high-purity water and in aqueous buffers, but unlike most research peptides it is itself an acid, so a concentrated stock in unbuffered water will be acidic. Either prepare the stock in a buffer of adequate capacity (for example 50 mM HEPES or phosphate at pH 7.2 to 7.4) and confirm the final pH, or prepare it in water and adjust with dilute sodium hydroxide; neutralizing converts the peptide to its sodium salt, which changes the mass per mole if it was weighed as the free acid. At 100% peptide content, 10 mg is 25.6 µmol (10 mg ÷ 390.35 g/mol), so 2.56 mL of solvent gives a 10 mM stock and 1 µg/mL is 2.56 µM; as a mono-trifluoroacetate salt the same 10 mg holds about 7.74 mg of peptide, or 19.8 µmol, some 23% less. Keep stocks in single-use aliquots at −20 °C or −80 °C, filtered through a 0.22 µm low-binding membrane for cell culture, and avoid repeated freeze–thaw cycles.
Chemical stability in solution. Epitalon carries no oxidation-prone residue (no methionine, cysteine or tryptophan), so it is comparatively indifferent to air. Its characteristic liability is the Asp–Gly bond: as Geiger and Clarke established for aspartyl and asparaginyl residues, the glycine backbone nitrogen attacks the aspartyl side-chain carbonyl to form a cyclic succinimide, which hydrolyses to a mixture of the α-aspartyl peptide and the β-aspartyl (isoaspartyl) isomer with partial racemization at that centre. The reaction is fastest at neutral to mildly alkaline pH, exactly where culture buffers sit, and much slower in the lyophilized solid, in acidic solution and at low temperature. So keep stocks frozen rather than refrigerated, prefer slightly acidic storage buffers to pH 8 ones, and regard long-stored aqueous solutions as candidates for re-analysis; because the two isomers share a mass, that check needs chromatography, not only a mass spectrum.
Verification. A short LC-MS run confirms identity and integrity: [M+H]+ at m/z 391.146, or [M−H]− at 389.131 in negative mode, with no peak 18 Da lower (373.135), which would indicate the succinimide form. Each lot's certificate of analysis, shown on this page, records the results for that lot.
Frequently Asked Research Questions
- What is Epitalon?
- Epitalon is the synthetic tetrapeptide L-alanyl-L-α-glutamyl-L-α-aspartyl-glycine, H-Ala-Glu-Asp-Gly-OH (AEDG), also called Epithalon, Epithalone or the AEDG peptide. Molecular formula C14H22N4O9, average molecular weight 390.35 g/mol, monoisotopic mass 390.1387 Da.
- What are the CAS number and PubChem CID of Epitalon?
- Epitalon is registered under CAS number 307297-39-8 and appears in PubChem as compound 219042. Its FDA Unique Ingredient Identifier is O65P17785G and its ChEBI identifier is 230091.
- Is Epitalon acidic or basic?
- Strongly acidic: three carboxyl groups (C-terminus, aspartic and glutamic acid side chains) outnumber the single N-terminal amine, giving a calculated isoelectric point of about pH 3.0 to 3.7 and a net charge near −2 at pH 7.4, unusual among research peptides, which are mostly cationic at neutral pH.
- What masses should I see for Epitalon by mass spectrometry?
- Positive-mode electrospray gives [M+H]+ at m/z 391.146, with sodium and potassium adducts at 413.128 and 429.102 and a weak [M+2H]2+ at 196.077 (only one basic site). Negative mode gives [M−H]− at 389.131. Diagnostic fragments: b3 316.114 with y1 76.039, and y3 320.109.
- What is the Asp–Gly problem, and why does it matter for this peptide?
- In an Asp–Gly sequence the unhindered glycine amide nitrogen closes onto the aspartyl side chain to form a succinimide (aspartimide), which reopens to give the β-aspartyl (isoaspartyl) isomer and partly racemized material. Repeated piperidine steps drive it during Fmoc synthesis, where Asp–Gly is the most susceptible sequence and the model Mergler and colleagues used to test countermeasures, and the same chemistry proceeds slowly in stored solutions near neutral pH. The isomers share the parent mass, so detecting them needs chromatographic or chiral analysis.
- What is the difference between purity and peptide content for Epitalon?
- HPLC purity is the fraction of UV-absorbing material that is the target peptide; peptide content is the fraction of the weighed powder that is peptide rather than counterion, water or salt. A mono-trifluoroacetate salt has a formula weight of 504.37 g/mol and so is at most 77.4% peptide by weight.
- How do I prepare a 10 mM stock from 10 mg?
- 10 mg ÷ 390.35 g/mol = 25.6 µmol, so 2.56 mL of solvent gives 10 mM at 100% peptide content, and 1 µg/mL is 2.56 µM. Correct for the peptide content on the lot's certificate of analysis, and check the pH of the concentrated stock, since the free peptide is itself an acid.
- Which in vitro assays are used to study Epitalon and telomerase?
- Telomere length by quantitative PCR as a telomere-to-single-copy-gene ratio (Cawthon); hTERT mRNA by RT-qPCR; telomerase activity in lysates by the telomeric repeat amplification assay (TRAP), with a heat-inactivated negative control and a telomerase-positive reference; and, for the telomerase-independent ALT pathway, the C-circle assay of Henson and colleagues with PML-body immunofluorescence. The 2025 study by Al-Dulaimi and colleagues applied all four.
- What concentrations and exposure times appear in the in vitro literature?
- The 2025 telomere study used 0.1 to 1.0 µg/mL (0.26 to 2.6 µM) for 4 days in cancer lines and 1.0 µg/mL for 3 weeks in fibroblast and epithelial cultures, with daily addition; in the fibroblast strain a 4-day exposure changed nothing, so the interval matters in slowly dividing cultures. Molar conversion: 1 µg/mL is 2.56 µM for the free peptide.
- How should Epitalon be stored?
- The lyophilized solid tightly closed at −20 °C away from light and moisture, warmed in a desiccator before opening; solutions in single-use aliquots at −20 °C or −80 °C, avoiding repeated freeze–thaw cycles and prolonged storage at neutral to alkaline pH, which favours succinimide formation at the Asp–Gly bond.
Sources & Further Reading
- National Center for Biotechnology Information. PubChem Compound Summary for CID 219042, Epitalon. PubChem CID 219042.
- Khavinson VKh, Bondarev IE, Butyugov AA. Epithalon peptide induces telomerase activity and telomere elongation in human somatic cells. Bulletin of Experimental Biology and Medicine 2003;135(6):590–592. doi:10.1023/A:1025493705728
- Al-Dulaimi S, Thomas R, Matta S, Roberts T. Epitalon increases telomere length in human cell lines through telomerase upregulation or ALT activity. Biogerontology 2025;26(5):178. doi:10.1007/s10522-025-10315-x
- Al-Dulaimi S, Thomas R, Matta S, Roberts T. Correction: Epitalon increases telomere length in human cell lines through telomerase upregulation or ALT activity. Biogerontology 2026;27(1):1. doi:10.1007/s10522-025-10326-8
- Araj SK, Brzezik J, Mądra-Gackowska K, Szeleszczuk Ł. Overview of Epitalon: highly bioactive pineal tetrapeptide with promising properties. International Journal of Molecular Sciences 2025;26(6):2691. doi:10.3390/ijms26062691
- Khavinson V, Diomede F, Mironova E, et al. AEDG peptide (Epitalon) stimulates gene expression and protein synthesis during neurogenesis: possible epigenetic mechanism. Molecules 2020;25(3):609. doi:10.3390/molecules25030609
- Fedoreyeva LI, Kireev II, Khavinson VKh, Vanyushin BF. Penetration of short fluorescence-labeled peptides into the nucleus in HeLa cells and in vitro specific interaction of the peptides with deoxyribooligonucleotides and DNA. Biochemistry (Moscow) 2011;76(11):1210–1219. doi:10.1134/S0006297911110022
- Fedoreyeva LI, Smirnova TA, Kolomijtseva GYa, et al. Interaction of short peptides with FITC-labeled wheat histones and their complexes with deoxyribooligonucleotides. Biochemistry (Moscow) 2013;78(2):166–175. doi:10.1134/S0006297913020053
- Rogachevskii IV, Shchegolev BF, Khavinson VKh. Geometric structure of a molecule of Epitalon tetrapeptide: a molecular-dynamics simulation. Russian Journal of General Chemistry 2006;76(5):826–831. doi:10.1134/S1070363206050276
- Greider CW, Blackburn EH. Identification of a specific telomere terminal transferase activity in Tetrahymena extracts. Cell 1985;43(2):405–413. doi:10.1016/0092-8674(85)90170-9
- Kim NW, Piatyszek MA, Prowse KR, et al. Specific association of human telomerase activity with immortal cells and cancer. Science 1994;266(5193):2011–2015. doi:10.1126/science.7605428
- Cawthon RM. Telomere measurement by quantitative PCR. Nucleic Acids Research 2002;30(10):e47. doi:10.1093/nar/30.10.e47
- Henson JD, Cao Y, Huschtscha LI, et al. DNA C-circles are specific and quantifiable markers of ALT activity. Nature Biotechnology 2009;27(12):1181–1185. doi:10.1038/nbt.1587
- Mergler M, Dick F, Sax B, Weiler P, Vorherr T. The aspartimide problem in Fmoc-based SPPS. Part I. Journal of Peptide Science 2003;9(1):36–46. doi:10.1002/psc.430
- Subirós-Funosas R, El-Faham A, Albericio F. Aspartimide formation in peptide chemistry: occurrence, prevention strategies and the role of N-hydroxylamines. Tetrahedron 2011;67(45):8595–8606. doi:10.1016/j.tet.2011.08.046
- Geiger T, Clarke S. Deamidation, isomerization and racemization at asparaginyl and aspartyl residues in peptides: succinimide-linked reactions that contribute to protein degradation. Journal of Biological Chemistry 1987;262(2):785–794. doi:10.1016/S0021-9258(19)75855-4
- Merrifield RB. Solid phase peptide synthesis. I. The synthesis of a tetrapeptide. Journal of the American Chemical Society 1963;85(14):2149–2154. doi:10.1021/ja00897a025
- Carpino LA, Han GY. 9-Fluorenylmethoxycarbonyl amino-protecting group. The Journal of Organic Chemistry 1972;37(22):3404–3409. doi:10.1021/jo00795a005
- Wysocki VH, Tsaprailis G, Smith LL, et al. Mobile and localized protons: a framework for understanding peptide dissociation. Journal of Mass Spectrometry 2000;35(12):1399–1406. doi:10.1002/1096-9888(200012)35:12<1399::AID-JMS86>3.0.CO;2-R
Last reviewed:
In the research library
Everything the library holds on Epitalon, and the methods behind the numbers on its certificate.
- Epitalon reference entry Identity, calculated properties, the mass spectrometry ions to expect and analytical notes, from the structure.
- Check a certificate against this sequence Paste the masses from a spectrum or a certificate; the mass-match tool compares them with what this sequence should give.
- Peptide calculator, with this sequence Formula, average and monoisotopic mass, charge across pH, isoelectric point and absorbance, recalculated as you edit.
- How to read a certificate of analysis What a peptide certificate of analysis should contain, how to check that it belongs to the material in hand, how to read its identity and purity results, and the signs that it deserves a second look.
- HPLC purity analysis of peptides How reversed-phase HPLC measures the chromatographic purity of a peptide, what the figure includes, and what it leaves out.
- Mass spectrometry for peptide identity How mass spectrometry confirms that a peptide is the intended sequence: electrospray and MALDI, working out the expected mass, reading charge states and adducts, sequence confirmation, and the limits of the method.
- Net peptide content and purity: two different numbers Why a peptide that is 99% pure by HPLC can be only 75–85% peptide by weight: what the powder contains, how each part is measured, and how the two figures combine.
- Preparing peptide solutions in the laboratory From a freeze-dried vial to a solution of known concentration: the arithmetic, the solvent, the charge chemistry and the handling, with the errors each step can introduce and the article that covers it.
- Peptide stability and storage How peptides degrade, chemically and physically, why the dry solid lasts far longer than a solution, which sequences are most at risk, and the storage and handling that slow it down.